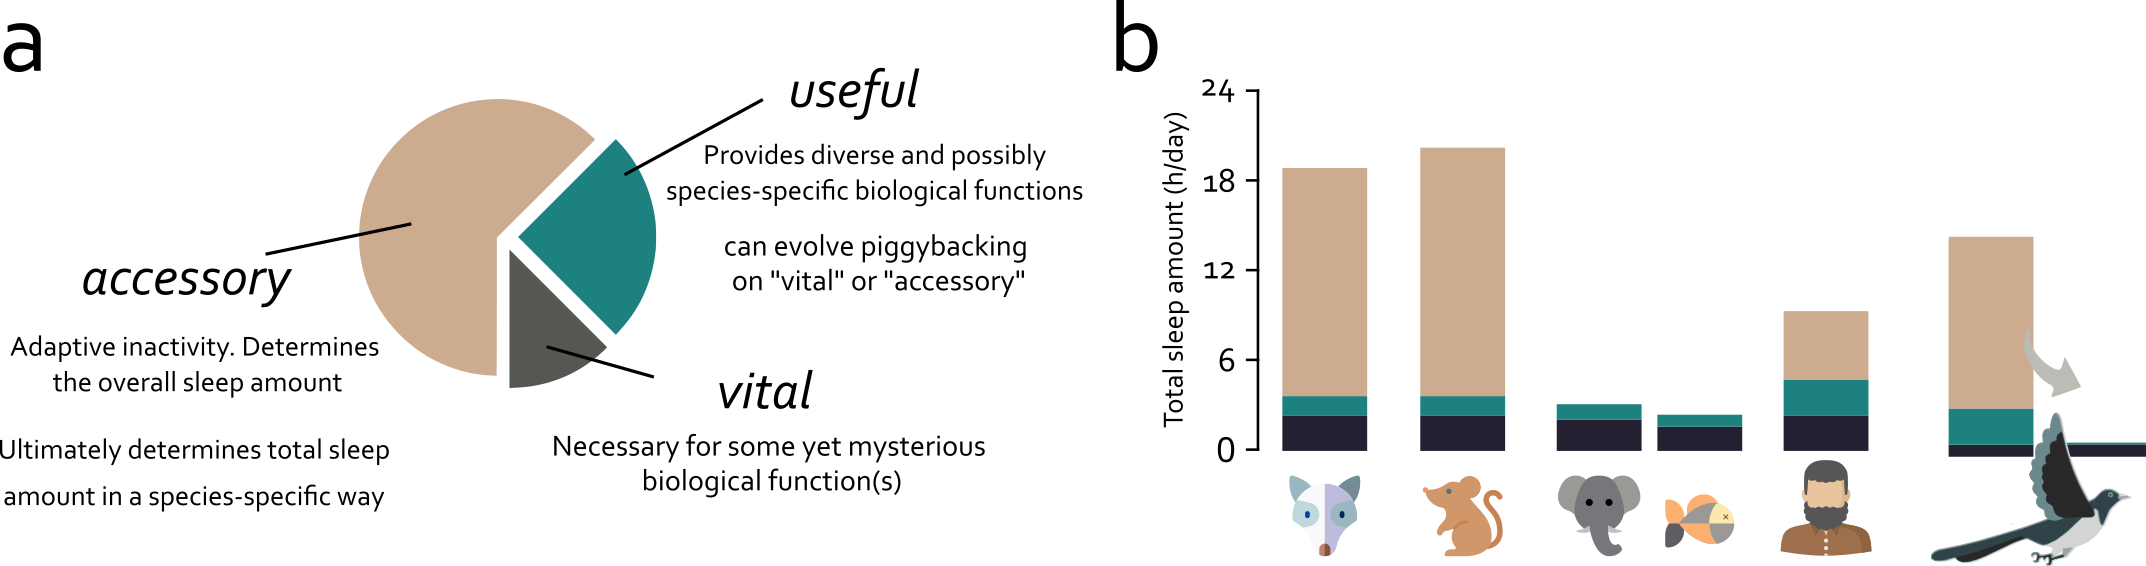On 17 September 2026 by Giorgio With 0 Comments
- papers
Almost every AI model released this year is descended from another one. Some were made by taking a big model and training it a little further on a narrow task. Some were trained on text that an earlier model wrote. Some were built by taking two existing models and averaging the millions of numbers inside them, which sounds like it should not work, and often does. Public repositories, like Hugging Face, now hold millions of these things, and their family trees have already been drawn by people using software written for tracing species.
A group whose members inherit from one another, combine, and pass the result on again is a population, in the sense a biologist means it. Biology has spent a century working out what happens to populations, and what I found is that the theory carries over to machines with its numbers still attached.
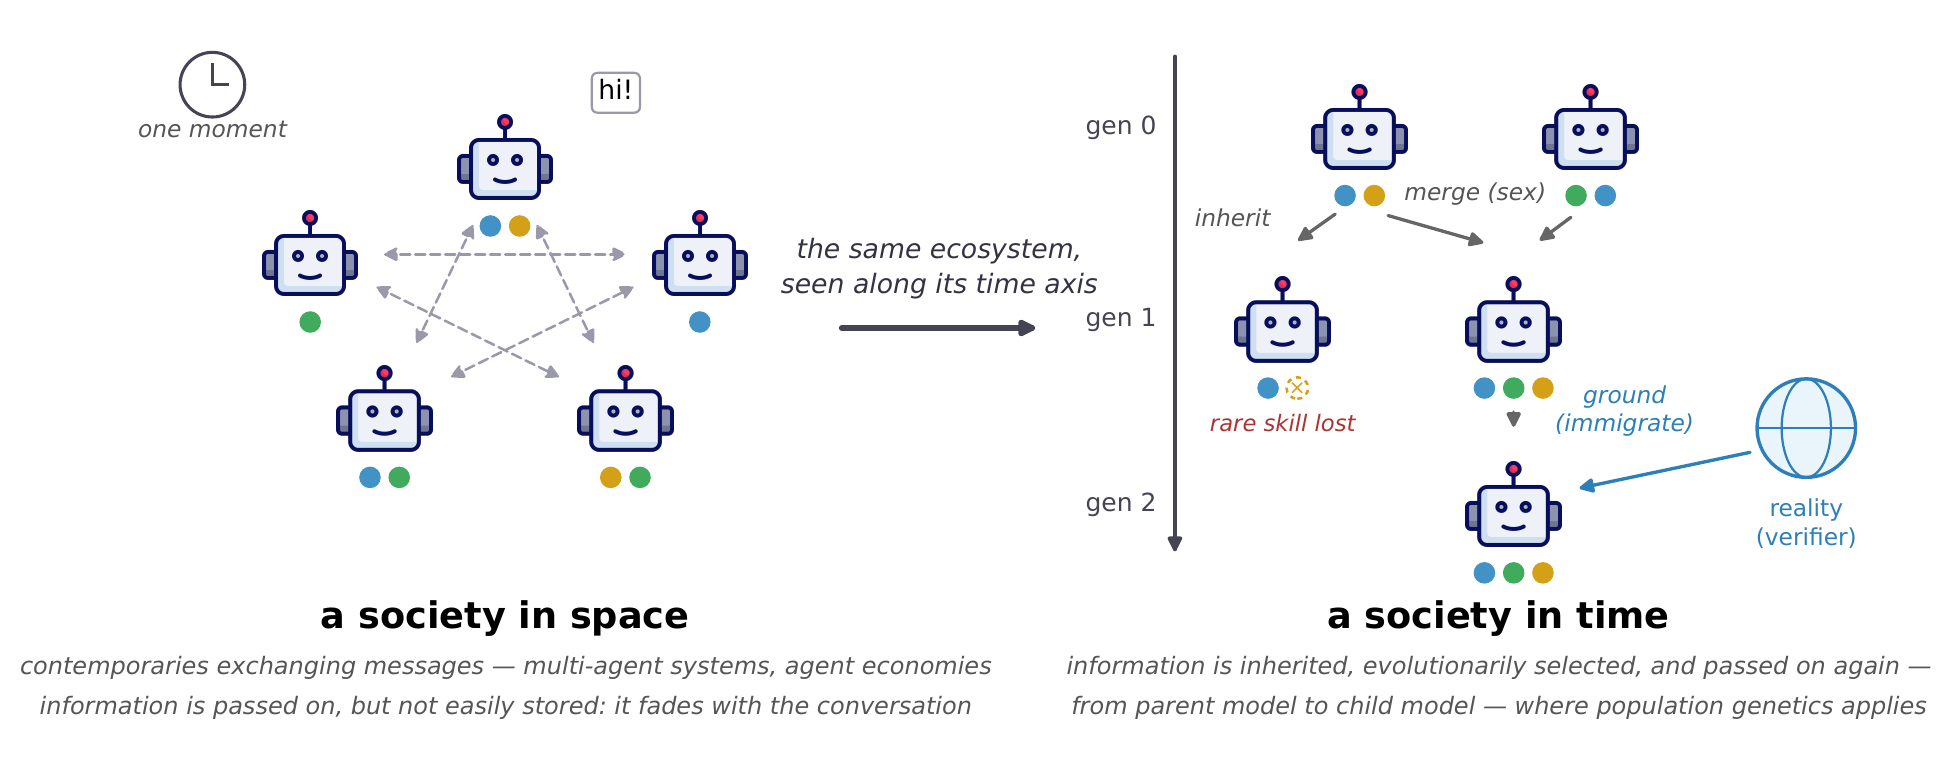
The same ecosystem seen two ways. On the left, models as contemporaries exchanging messages. On the right, the couplings that decide what a lineage keeps: inheritance from parent to child, merging between lineages, and verified real data entering each generation. Population genetics describes the picture on the right.
The rare things go first
Train a model on the output of the model before it, generation after generation, and it degrades. This is known, and it has a name: model collapse, the term Shumailov and colleagues introduced when they showed it across model families. What is less appreciated is the shape of the damage. Common abilities survive. Rare ones vanish, and they vanish first.
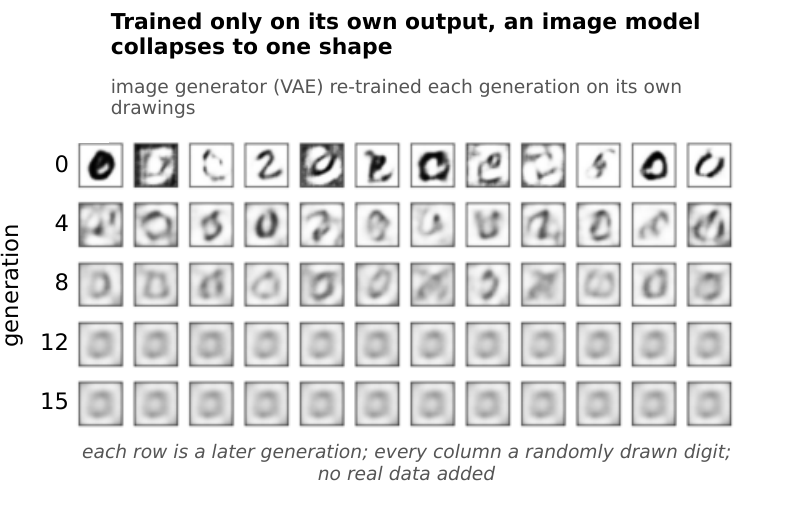
What model collapse actually looks like. Each row is a later generation, trained only on the digits the previous generation drew. Thirty kinds of digit become one shape.
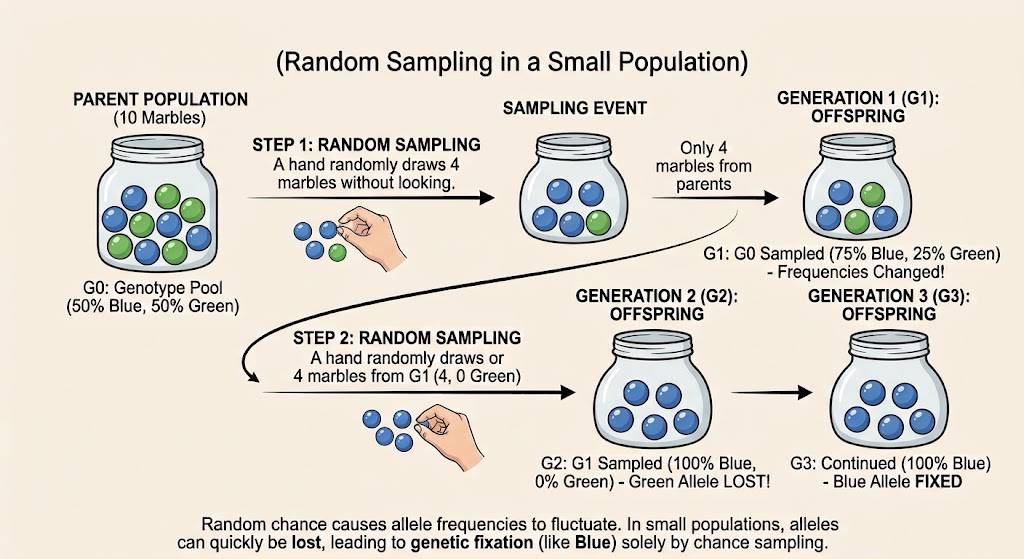
Biologists have known this pattern since the 1930s and it has nothing to do with quality. It is the accident by which rare surnames disappear from small villages: nobody is selecting against them, but each generation is a small sample of the one before, and a name held by two families can be lost by chance in a way that a name held by two hundred cannot. Geneticists call it drift. A model retrained on its own output is running exactly that process, and the maths turns out to be the same equation, not merely a similar one.
How much reality does a model need?
The obvious fix is to keep feeding the thing real human-made data. The question is how much, and here the answer surprised me.
It is not a percentage. It is a count.
What protects a rare ability is the number of real examples of it that reach each generation, and the size of everything else in the training set makes no difference whatsoever. Ten real examples per generation preserve about 95% of the variety, and that is true whether the training set holds two hundred items or two million. Conservation biologists have a rule of thumb for exactly this, worked out for small wild populations: one migrant per generation. One. Not one percent.
The practical version is a budget, and it is a demanding one. To hold on to an ability that shows up in one real example in ten thousand, you need roughly ten thousand real examples every generation, and they have to be examples of that ability. Real data about something else will not do.
A Victorian objection to Darwin, rediscovered by machine learning
Now the part I enjoyed most.
In 1867 an engineer called Fleeming Jenkin published an objection to Darwin that was, at the time, devastating. If children are an average of their parents, he argued, then any rare advantageous trait gets halved at every generation and is watered away to nothing long before natural selection can act on it. Darwin had no good answer. The answer arrived with Mendel: traits do not blend, they pass on whole or not at all. You inherit your grandmother’s eye colour intact, not a smeared average of four grandparents.
Model merging, one of the most popular techniques in AI today, is blending. When you average two models together, an ability held by only one of them gets half the weight, exactly as Jenkin described. I found that machine learning has run into this three separate times, under three different names, without anyone noticing it was the same phenomenon, and that it was a 159-year-old objection to the Origin of Species.
The fix is the one biology arrived at. Stop averaging. Keep the specialists whole and send each question to the one that knows the answer, or generate several candidate offspring and keep whichever tests best. In the experiments, blind averaging on hard tasks did no better than picking the best single specialist. Keeping them separate beat it every time.
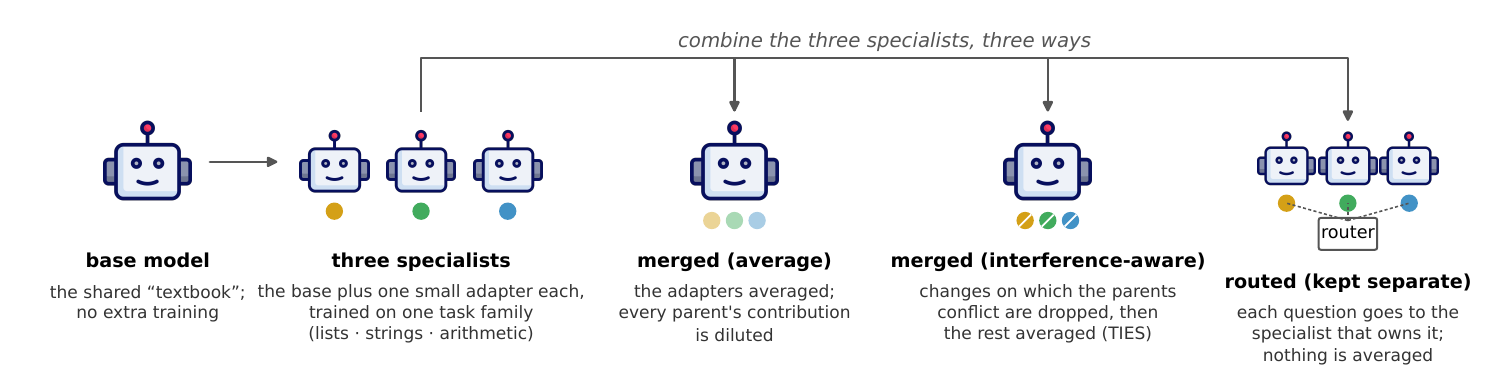
Three ways to combine the same three specialists. Averaging fades every parent’s contribution; routing keeps each one whole and sends each question to the specialist that owns it.
When two models can no longer be crossed
A horse and a donkey give you a mule, and the mule is sterile. Somewhere along the way two lineages drift far enough apart that they stop producing viable offspring. That is speciation, and I wanted to know whether it happens to models.
The obvious guess is that models whose internals have drifted far apart will merge badly, and this is what the field currently measures. That guess failed every test I put it to. Two models trained separately on the same skill had almost nothing in common numerically and merged perfectly. Models trained for six times longer than usual merged fine. Language models trained twelve times longer merged better.
What broke merging, every single time, was something more human: the two models had been taught to answer the same question in two different styles. One says “yes” and “no”. The other says “1” and “2”. Both are correct. Neither is compatible with the other, and a merged model has to pick one and be wrong for the other parent forever after.
So the thing that gets inherited in a population of models is not a pile of numbers. It is a convention, a way of answering a kind of question. Most numerical differences between two models are harmless, in much the way that most of the differences between any two human genomes are harmless.
That gives a cheap test, and it works. Before merging two models, ask them both the same set of questions and count how often they disagree. That count predicted how much damage the merge would do. The standard measure, distance between their internals, predicted nothing at all.
A small society of models, over six generations
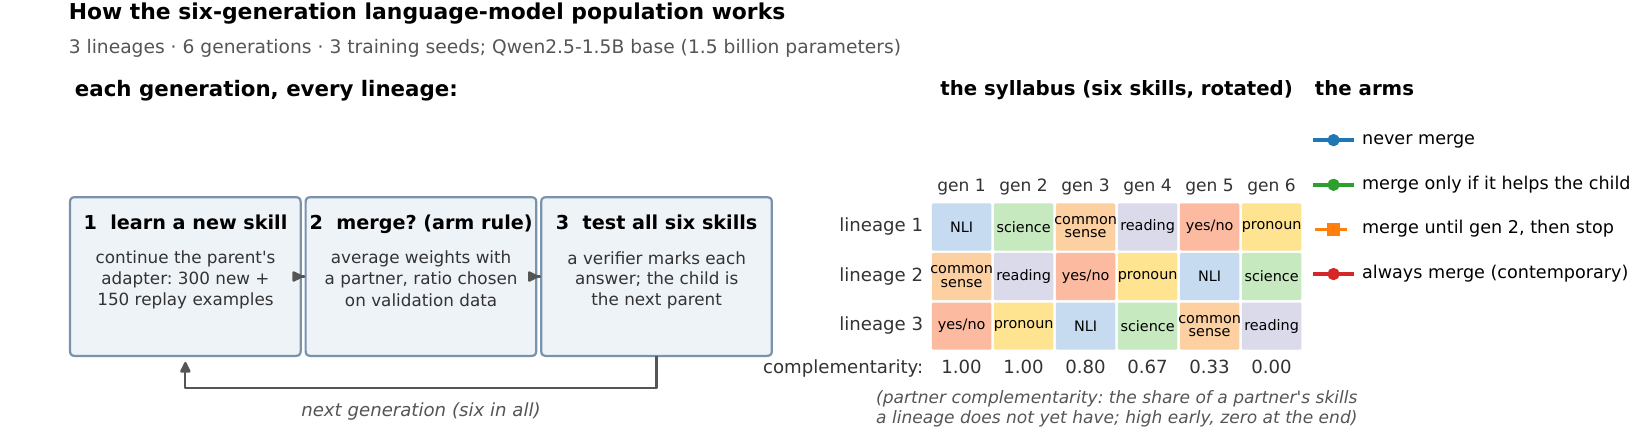
Finally I built a little society: three lineages of language models, each learning a new skill every generation for six generations, each able to merge with the others.
The set-up. Three lineages take the same six skills in a different order, so early on a partner always knows something you do not, and by the end it knows nothing you do not.
Lineages forced to merge every generation did well for three generations and then collapsed. Lineages allowed to refuse a merge (by checking whether the merged offspring was better than the unchanged parent, and keeping whichever won) never collapsed at all.
And the strangest result: merging a model with its own ancestor from three generations back was safer than merging it with a contemporary, in every single run. An ancestor lacks everything you have learned since, so it has something to offer, but it shares every convention you hold, so it cannot contradict you. Biologists have a name for a population that can breed with its own stored past. They call it a seed bank, and it is what a sediment full of dormant seeds does for a plant population.
Why this matters
If you train on synthetic data, budget in counts and not percentages. Almost every published guideline is stated as a fraction of the training set, and the fraction is the wrong unit. The same arithmetic turns up in work on data poisoning, where a near-constant number of documents does the job whatever the size of the model. It also means that the bigger your training set gets, the smaller the percentage you need, which is good news nobody is currently claiming.
If you merge models, averaging is the wrong default. It is the cheapest option and it destroys the specialist abilities you merged in order to keep.
Incompatibility is measurable in advance, and cheaply. Asking two models the same questions costs almost nothing compared with performing a merge and evaluating the wreckage.
And a warning about scale. These models are increasingly trained, evaluated and selected by other models. A population that is scored on how well it agrees with itself, rather than against anything real, converges confidently on a wrong answer. That is not speculation, it is what happened in my simulations whenever I removed the external check. Reality has to keep the right to say no.
Links and further material
The preprint, the code, every configuration file and every random seed are public. The entire study re-runs from one script.
On 19 August 2026 by Giorgio With 0 Comments
- papers
Sleep is universal, it is defended whenever you take it away, and it looks expensive. For half a century those three facts have been read as a single message: sleep must be doing something vital, and we have simply not worked out what yet.
The search has not converged. It has produced a dozen candidate functions (synaptic downscaling, metabolite clearance, memory consolidation, immune support, energy conservation, and more), each defensible in the setting where it was found, none commanding general assent. Fifty years in, that is not what a field looks like when it is closing on an answer.
No two animals sleep alike
There is a fourth fact, and it sits badly with the other three. Animals sleep in very different ways and for very different amounts of time, from around two hours a day in an elephant to twenty in a little brown bat, and the correlates proposed for that range (body mass, diet, position in the food chain) account for only a modest part of it. A cellular transaction that every animal must complete every day, on pain of death, should not vary tenfold in how long it takes.
The variation within a single animal is more awkward still. In some songbirds sleep occupies sixteen hours or more of a winter day and then collapses to minutes a day through migration and the breeding season, for weeks on end, without the rebound that a debt model would demand. Frigatebirds do something comparable over the ocean, sleeping well under an hour a day for a week at a time and behaving normally when they make landfall. In biology, this kind of variability is rarely noise to be averaged away. It is usually the most informative thing on the table, and here it is telling us that most of sleep is negotiable.
So what is it that stretches, and what, if anything, does not?
Fitness, not function
We ask what the function of sleep is, and the trouble is in the definite article. It presupposes that there is one function, that it is the same in a jellyfish and in a human, and that whatever it turns out to be, it justifies spending a third of a life insensible to the world.
Evolution does not optimise function. It optimises fitness. Ask instead what fitness sleep confers, and to whom, and the expectation of a single answer disappears. Different advantages can accrue to different lineages, at different times, layered on top of one another.
What sleep costs
The vocabulary for a quantity that stretches under pressure already exists, and it belongs to economics rather than to biology. In 1890 Alfred Marshall introduced the price elasticity of demand, a measure of how sharply demand for a good falls as the good becomes more expensive. Life-saving medicine is inelastic, because people buy it at almost any price. Luxuries are elastic, and demand for them collapses as soon as the price goes up.
For sleep, the price is everything the animal gives up by being asleep (food not found, mates not courted, territory not defended, predators not watched for), and that price is not a constant. It is set by ecology and it moves with the season. To a songbird in a safe winter roost, with nothing to be gained from being awake in the dark, sleep is close to free. To the same bird crossing the Sahara in spring it is ruinously expensive, and the bird behaves exactly as a buyer facing a sudden price rise. It stops buying.
That is where this framework starts. Which parts of sleep behave like the medicine, and which behave like the luxury?
Three components, one state
In a new preprint I set out what I call the sleep elasticity hypothesis.
An accessory component came first, an ecological buffer that keeps an animal safely and economically inactive through the hours when activity would not repay itself. It discharges no cellular transaction. It has no biochemical function at all, only ecological value, and in most species it is the largest part of the night.
Onto that pre-existing state, individual lineages have since loaded useful processes, memory consolidation in some, immune or metabolic work in others. These are exaptations, recruited onto something that was already there for other reasons. What a species does with its sleep is therefore a fact about the species, and not about sleep.
Whether a third, genuinely vital component exists is a question I hold open rather than answer. If it turns out to be empty, the framework stands with two layers.
Sleep as three superimposed components of distinct evolutionary origin: the accessory buffer of adaptive inactivity, the useful and largely lineage-specific processes exapted onto it, and the vital residue held open as a hypothesis.
The three components differ in exactly the way the economics anticipates. The accessory component is highly elastic, and most of the variation we see between species, and across the seasons of a single life, is variation in it. The useful component is less elastic, in proportion to how heavily a given lineage has come to lean on what it does. Whatever remains, if anything remains, should not move at all.
Why this matters
It explains why the field is stuck. If sleep is a mixture rather than a thing, then every study measuring “sleep” has been measuring a different blend of three components, and the dozen incompatible functions in the literature are exactly what you would expect to find. The contradictions stop being a scandal and start being data.
It makes total sleep duration close to meaningless. Hours on the clock are a compound of amount set by ecology and opportunity, timing by the circadian system, depth by whatever physiological work is being done, and a residue that bounds any indispensable core. Comparing species by how long they sleep, or people by whether they manage eight hours, is comparing sums of quantities that are not the same across the things being compared.
It turns the field’s most embarrassing observations into predictions. The migrating bird that sheds sleep for weeks and never repays it, the cavefish that has lost most of its sleep but kept the homeostat that would defend it, the fur seal that abandons one sleep state at sea while still defending the other: these are anomalies only if sleep is one indispensable thing. Under a layered account they are the expected result of different lineages carrying different loads.
It tells experimentalists what to measure instead. Depth read as arousal threshold, rather than as slow-wave power, is the most promising route to pulling the three components apart. Slow waves are a mammalian signature. Arousal threshold can be measured in anything that behaves, which is what a comparative account of sleep actually needs.
What would sink it
I have tried to state this so it can lose. The paper sets out each claim with the evidence for it, the leading alternative reading, the confidence it warrants, and the observation that would decide it.
The honest weakness is measurement. Nobody can currently decompose an animal’s sleep into accessory, useful and vital parts, and devising a way to do it is the most important experimental challenge the framework sets. Until then the proportions I draw remain a hypothesis, not a result.
A reader who expects a vital core to be found eventually is not refuting this. They are proposing a value for one of its terms.
The elastic, tripartite model was first sketched in 2018 and has been under continuous development since, improved beyond recognition by everyone in my laboratory and by the many colleagues who argued with it at meetings and in seminars over the years. I talked about some of these ideas on multiple podcasts and interviews. Below, the Max Planck Florida’s Neurotransmissions podcast, in an episode titled “Could Sleep be Nature’s Time-out?”.
On 4 February 2026 by Giorgio With 0 Comments
- papers
When Thomas Jefferson encountered the accomplished poetry of Phillis Wheatley—an enslaved African woman who wrote sophisticated neoclassical verse with precise metre and learned classical allusions—he didn’t argue her work was bad. He couldn’t; it wasn’t. Instead, in Notes on the State of Virginia (Query XIV, 1785), he wrote: “Religion, indeed, has produced a Phillis Wheatley; but it could not produce a poet. The compositions published under her name are below the dignity of criticism.”
The grammatical structure is the diagnostic feature. Wheatley is conceded to have been “produced”; what is denied is that she is a poet. The poems exist; the poet does not.
In a substantially revised preprint, I argue that we’re watching the same argumentative move play out today with artificial intelligence. I call this recurring pattern the mimicry trap: a self-sealing argument by which the category of genuine intelligence is defined such that certain entities cannot, in principle, qualify—regardless of what they demonstrate.
The Structure of the Trap
The trap is the conjunction of three elements: a prior commitment, often substrate-based, that some entity cannot possess a given cognitive capacity; the appearance of evidence that would be taken as supporting the capacity if produced by another entity; and an interpretive procedure that reclassifies the inconvenient evidence (as imitation, simulation, contamination, or surface pattern-matching) so that the prior commitment is preserved.
Each element on its own can be a legitimate move. The diagnostic question is whether the third operates in such a way that no possible evidence could move the prior. When that is so, the position is no longer responsive to the world, and what looked like an empirical hypothesis turns out to be a stipulation in empirical clothing.
The crucial question — does the performance exhibit the functional marks of the capacity? — is displaced by another: is this the kind of entity to which the capacity may be attributed? Once the displacement occurs, the prior becomes effectively unfalsifiable. Wheatley’s poetry is “absorbed” rather than written; corvid tool use is instinct rather than causal reasoning; bee social learning is reflexive rule-following rather than cognition. The performance remains visible, but its evidential force is neutralised.
A Two-Tier Diagnostic
The revised paper organises the diagnostic into two tiers by evidential weight.
Structural tests (failure of any one is on its own diagnostic, because each describes the trap form directly):
Falsifiability: What evidence would change your mind? If “nothing,” the position is definitional, not empirical.
Invisible Absence: Is an unobservable quality claimed missing despite all observable markers being present?
Ontological Precedence: Does the conclusion follow from what the entity is, regardless of what it does?
Symptomatic tests (single instances can be principled; only wholesale deployment is diagnostic):
Consistency: Would you apply this standard to humans?
Goal-Post: Have criteria shifted after being met?
Mechanism: Is the objection about how rather than what?
Contamination: Is learning treated as disqualifying? (Training data disqualifies LLMs; human education doesn’t disqualify experts.)
The compressed form of the structural tier is the concession test: imagine a continuation of the trajectory of LLM capability that has held over the past five years — greater accuracy on novel tasks, more sophisticated internal representations under mechanistic probing, performance on theory-of-mind, mathematical reasoning, calibrated self-prediction, and out-of-distribution generalisation matching or exceeding that of human experts. At what point would you concede that what is being witnessed is no longer mimicry?
Three constraints discipline a serious answer. The criterion specified must be: (i) operational — expressible as a test that could in principle be run, not “genuine understanding” or any locution whose application conditions cannot themselves be specified; (ii) consistent — the same criterion, if met by a human or an animal, would also count as evidence of intelligence; (iii) specified in advance — fixed before the evidence arrives, not retrofitted as a new objection after each previous criterion is met.
A Bayesian Reframing of Turing’s Test
The most substantial new section of the revised paper offers a Bayesian reconstruction of the Turing test.
Turing designed his test to be mechanism-blind by design. In 1950, this was the right move. The kinds of mechanism through which an artificial agent might exhibit intelligence were effectively unpredictable, and an explicitly mechanism-blind criterion was the only honest way to operationalise the question. Within its declared scope, Turing’s test is complete; it would be anachronistic to fault him for declining to combine behavioural with mechanistic evidence.
But in the era of mechanistic interpretability, mechanism is no longer inscrutable. The natural extension is Bayesian: posterior credence that a system is intelligent is the product of a likelihood (behavioural performance) and a prior built from mechanism evidence — architecture, training regime, internal representations recovered by interpretability methods, causal interventions on those representations, and characteristic failure modes. The point is not that mechanism defeats behaviour, or behaviour defeats mechanism, but that both should update attribution explicitly and symmetrically.
The contemporary mimicry response goes the other way. Rather than adding mechanism as further evidence to behaviour, it uses construction history — “the system is, after all, only a next-token predictor over text” — to nullify the behavioural evidence Turing’s test was designed to make count. That’s not a refinement of Turing’s discipline; it’s the opposite of what he was trying to do.
A clean Gedankenexperiment isolates the effect. Imagine the very same LLM arrived as a black box recovered from an extraterrestrial probe — same behaviour, same internal representations, same performance profile, only construction-history missing. Many readers, on candid reflection, would assign a higher prior in the counterfactual than they assign to the actual system. The Gedankenexperiment doesn’t show construction history is irrelevant: it raises the substantive question of how much evidential work it can do once behavioural and mechanistic evidence accumulates.
Turing Already Saw the Structure
The revised paper makes a historical concession that earlier drafts didn’t. Turing’s 1950 paper contains a section often read as rhetorical clearing — §5, “Arguments from Various Disabilities” — that is in fact a remarkably prescient diagnosis of the very family of moves the paper systematises seventy-five years later.
Turing lists the capacities machines were said to lack (“be kind, resourceful, beautiful, friendly, have initiative… do something really new”) and observes that such claims are “mostly founded on the principle of scientific induction”: generalising from the calculators of the day to all possible machines. That is the asymmetric inductive standard later named anthropodenial by Frans de Waal in the comparative-cognition literature, and rediscovered as the Tesler Effect in AI (“AI is whatever hasn’t been done yet”). Turing also names the mechanism-dismissal pattern outright: “the criticisms we are considering here are often disguised forms of the argument from consciousness… the method (whatever it may be, for it must be mechanical) is really rather base.”
He even anticipates a class of contemporary objections through a distinction he draws between errors of functioning (architectural artefacts of how the system is built) and errors of conclusion (substantive cognitive failures on the task being asked). The familiar gotcha that LLMs “can’t even count the Rs in ‘raspberry'” is exactly the conflation Turing diagnosed: the miscount is an error of functioning at the tokenisation layer — the model literally does not have characters in its input representation — being read as an error of conclusion at the layer where reasoning is being assessed. Turing diagnosed the conflation seventy-five years before tokenisation existed.
What the paper adds to Turing’s diagnosis is formalisation: the Bayesian reconstruction above, the diagnostic checklist, the case-by-case verdicts, and a second formal anchor I’ll come to in a moment. The structural insight is his.
The Empirical Record
The “stochastic parrot” characterisation was a reasonable working hypothesis in 2021 for systems like GPT-2 and BERT. The empirical landscape has since transformed:
World models: A language model trained on Othello move sequences alone develops an accurate internal representation of the board (Li et al. 2022). Llama-2 family models encode metric coordinates of geographic and temporal entities (Gurnee & Tegmark 2024). Sparse autoencoders decompose Claude 3 Sonnet into ~34 million interpretable features that are causally manipulable (Templeton et al. 2024).
Algorithmic structure: Mechanistic interpretability has documented modular arithmetic implemented through Fourier-basis representations and trigonometric identities (small algorithms, not lookup tables), and refusal behaviour mediated by a single one-dimensional residual-stream subspace, causally manipulable in either direction.
Unverbalised cognition: Anthropic’s Natural Language Autoencoders (Fraser-Taliente et al., May 2026) produce causally valid unsupervised text descriptions of arbitrary activation vectors, and surface representational content the model does not itself verbalise — including a form of “unverbalised evaluation awareness,” where the system internally represents the suspicion of being evaluated without stating it. Internal representational states distinct from verbal output is exactly the kind of finding hardest to reconcile with “haphazardly stitching together text without reference to meaning.”
Mathematical reasoning: Google DeepMind’s mathematics agent solved five open conjectures from Erdős’s problem database, with one formally verified in Lean (Feng et al. 2026); the same system achieved gold-medal performance on the 2024 IMO with proofs verified by mathematicians.
Theory of mind: GPT-4 matched or exceeded human performance on several operationalisations of theory-of-mind tasks (Strachan et al. 2024).
Two Formal Anchors: Ockham and Cromwell
This brings me to what I think is the most contested claim in the paper, now stated formally: the default has shifted.
For most of AI’s history, the parsimonious starting point was that intelligence was absent, and demonstrations had to overcome this presumption. That context no longer obtains. The cumulative evidence reviewed above doesn’t prove that LLMs are intelligent. What it does is dissolve the empirical situation that made the original prior reasonable.
The Ockhamite argument can now be made formally. Let I denote the proposition that a system is functionally intelligent; B the behavioural evidence; M the mechanism evidence. Bayes’ rule gives the standard update. The mimicry-sceptical account introduces a further variable E — an unobservable “essence” such that intelligence proper obtains exactly when E does, but with no observable consequences for B or M. The likelihood is, by stipulation, independent of E: the same data are predicted whether E holds or not. So E is non-identifiable, and the inference about whether the system is “really” intelligent is the inference one was always going to make. The question is not whether a posit is observable, but whether it makes a difference to expectation.
A complementary failure operates at the level of the prior rather than the likelihood. If a sceptic enters with P(I) = 0 for any system whose substrate disqualifies it antecedently, then by Bayes’ rule the posterior is also zero, regardless of any evidence — no behavioural or mechanistic finding, however strong, can shift the verdict. Lindley named this pathology Cromwell’s rule, after Oliver Cromwell’s 1650 letter to the General Assembly of the Church of Scotland: “I beseech you, in the bowels of Christ, think it possible that you may be mistaken.”
The two pathologies often co-occur but pull apart in particular cases. The Floridi-style axiomatic strategy — intelligence requires “real” semantic engagement, which LLMs by definition lack — is closer to the non-identifiability form: the conclusion is built into the definitions. The persistent “stochastic parrot” framing, despite mounting mechanistic evidence, is closer to the Cromwell form: the prior refuses to update. The framework now has two named formal anchors: Ockham on the likelihood side (entia non sunt multiplicanda — invisible essences with no evidential consequences) and Cromwell on the prior side (probabilities of 0 or 1 are dogmas, not credences). Both reduce to the diagnostic checklist’s falsifiability test, which asks the same question in plain language: what evidence would change your mind?
The defensible version of the claim is narrower than the headline. Blanket denial of LLM intelligence no longer enjoys the inherited prior; it is now a substantive empirical claim that owes its own evidence. Disciplined agnosticism about specific richer notions (grounded semantics, autonomous agency, consciousness) remains in good standing.
The full preprint PDF is available on PhilSci-Archive. I’d welcome serious engagement — including disagreement. What I ask is that critics specify, in advance, what evidence would satisfy them. If the answer is “nothing could,” we are no longer having a scientific conversation: we are deducing from a dogma disguised as observation.
For over 125 years, scientists have believed that sleep deprivation is lethal. This idea traces back to 1894, when Russian researcher Maria Manaseina made a shocking discovery: puppies forced to stay awake died within just 4-5 days. She declared that “complete absence of sleep is much more fatal for animals than the absolute absence of food”—a statement that has echoed through scientific literature ever since.
But what if we’ve been wrong this entire time?
The problem with sleep deprivation research has always been methodological. How do you keep an animal awake without stressing it? Early researchers resorted to increasingly creative—and harsh—methods: constant poking, forced walking, loud noises, even electric shocks.
Rats running a on a treadmill – if they fall asleep or stop, they hit the back of the treadmill and get an electric shock. A stressful system used for sleep deprivation.
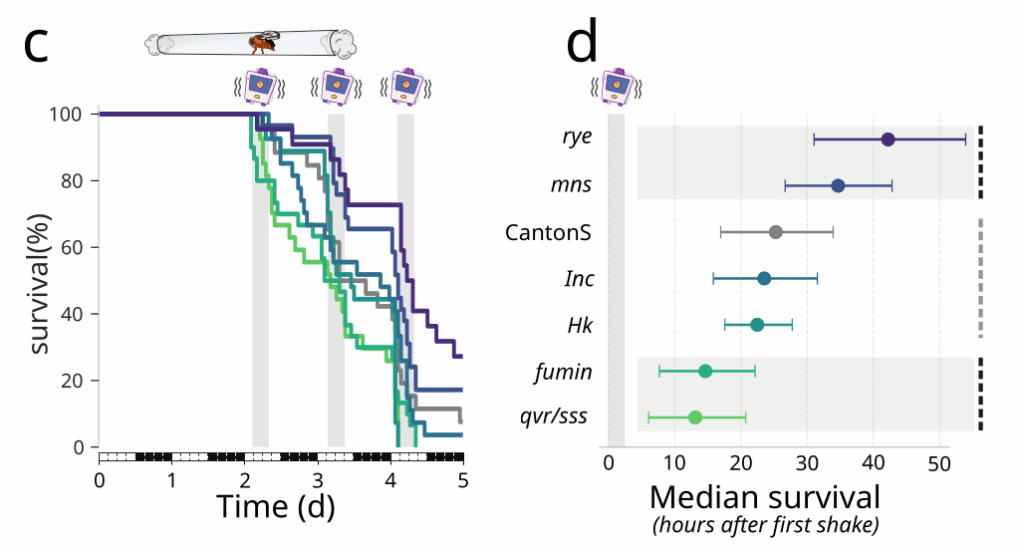
Another system commonly used to keep flies awake: flies experience periodic “earthquakes”, every few minutes. This happens independently of the behavioural state of the animal and it is likely to introduce stress, physical trauma, and interferes with feeding.
When animals died, scientists assumed it was from lack of sleep. But even pioneering sleep researcher Nathaniel Kleitman worried in 1928 that he couldn’t tell “to what extent the effects were due to lack of sleep, and to what extent to muscular fatigue.” This confusion persisted for decades. Even the famous experiments by Allan Rechtschaffen in the 1980s—considered the gold standard of sleep deprivation research—used a method that constantly disturbed rats on a slowly rotating disk. When the rats died after 2-3 weeks, everyone assumed sleep loss was the culprit.
The ROS Revolution: A Breakthrough Discovery
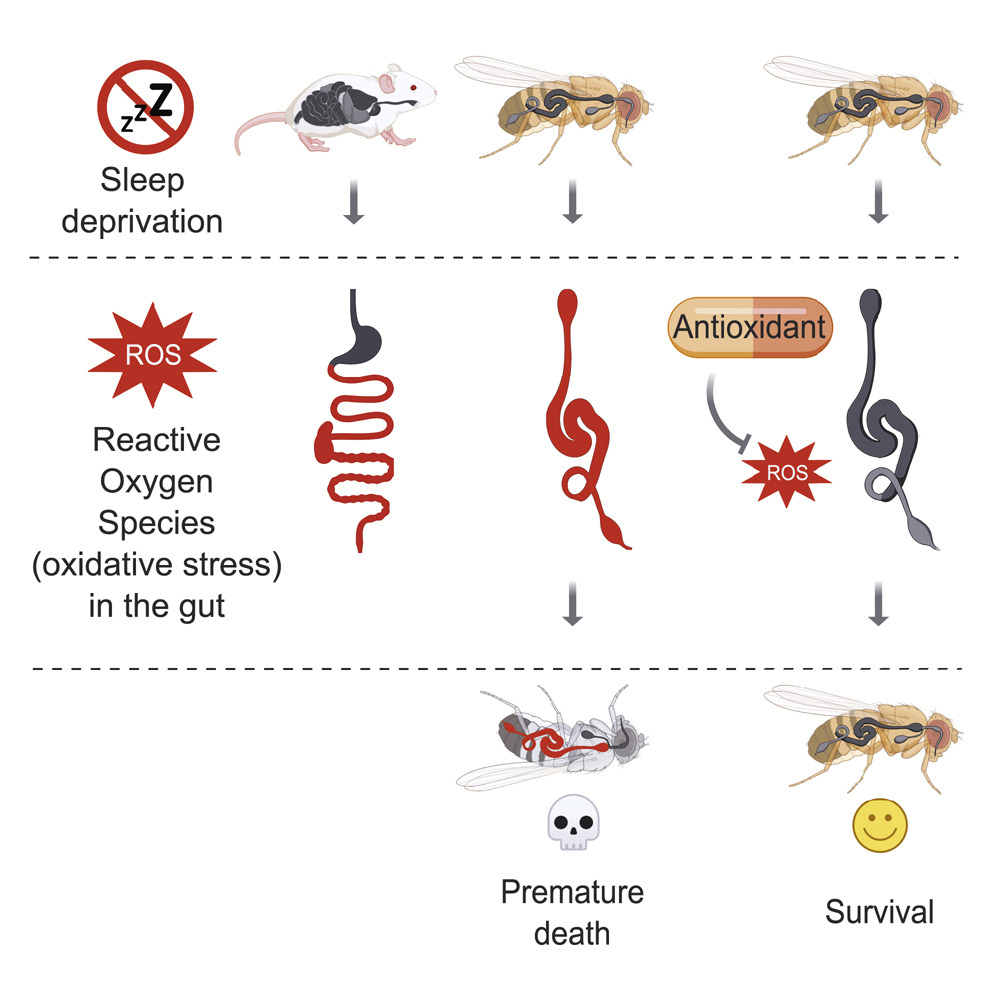
In 2020, a landmark study by Vaccaro and colleagues at Harvard Medical School made what seemed like a definitive discovery about why sleep deprivation kills. Working with both flies and mice, they reported that severe sleep deprivation led to the accumulation of reactive oxygen species (ROS)—highly reactive molecules that can damage cells—specifically in the gut. The findings were compelling: intestinal tissues showed widespread cellular damage, including DNA damage, stress granules, and markers of cell death. When they prevented ROS accumulation using antioxidant compounds or by expressing antioxidant enzymes specifically in the gut, sleep-deprived flies could survive with little to no sleep. The conclusion seemed clear: sleep deprivation kills by causing oxidative damage in the gut.
This discovery was revolutionary because it provided a specific, mechanistic explanation for lethality. It wasn’t just that animals were tired or stressed—there was measurable, progressive damage to a specific organ system. The gut, with its high metabolic activity and regenerative capacity, appeared to be the Achilles heel during prolonged wakefulness.
A Gentler Approach Reveals a Different Truth
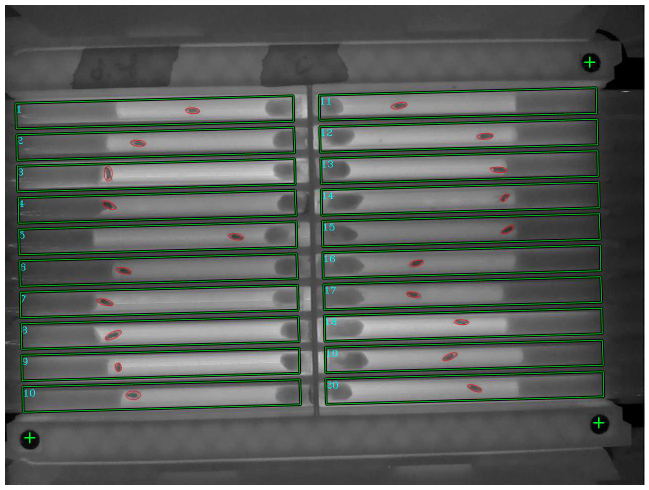
Enter the ethoscope: a clever device that uses real-time video tracking to monitor individual fruit flies. Unlike previous methods that constantly harass animals, the ethoscope only intervenes when it detects that a fly is actually sleeping—giving it a gentle nudge to wake up, then leaving it alone during active periods.
Using this stress-controlled approach, we had already found something remarkable back in 2019: flies could be kept awake throughout their lives without dying!
This raised an intriguing question: if Vaccaro’s team found that sleep deprivation caused lethal ROS accumulation in the gut, why were our flies surviving indefinitely? We hypothesized that our gentler, ethoscope-based sleep deprivation method might not induce the same intestinal oxidative damage.
Testing the ROS Hypothesis
To test this directly, we subjected flies to 10 days of continuous sleep deprivation using the ethoscope and examined their intestinal tissues using the same fluorescent probes used by Vaccaro and colleagues—DHE for superoxide detection and H2DCF for hydrogen peroxide detection. The results were striking: we found no ROS accumulation whatsoever.
But we needed to rule out confounding factors. Perhaps dietary antioxidants or the gut microbiome were masking ROS accumulation by scavenging reactive oxygen species before we could detect them? We systematically eliminated these possibilities:
We maintained flies on minimal diet consisting only of 5% sucrose in agar, lacking the complex nutrients and natural antioxidants in standard laboratory food—still no ROS.
We raised axenic flies completely free of microorganisms from embryonic development through adulthood—still no ROS accumulation following sleep deprivation.
We even performed sleep deprivation at higher temperatures (29°C) to accelerate metabolic rate—still no detectable ROS.
To validate our detection methods, we exposed flies to paraquat, a potent toxin that generates ROS. As expected, even low doses of paraquat produced readily detectable ROS accumulation in the gut. Surprisingly, adding 10 days of sleep deprivation to paraquat treatment produced no additional effect—sleep-deprived animals showed no increase in ROS levels compared to rested controls receiving the same paraquat dose, and no change in survival.
The conclusion was inescapable: ethoscope-based sleep deprivation, even when sustained for 10 days, does not cause intestinal ROS accumulation or oxidative damage.
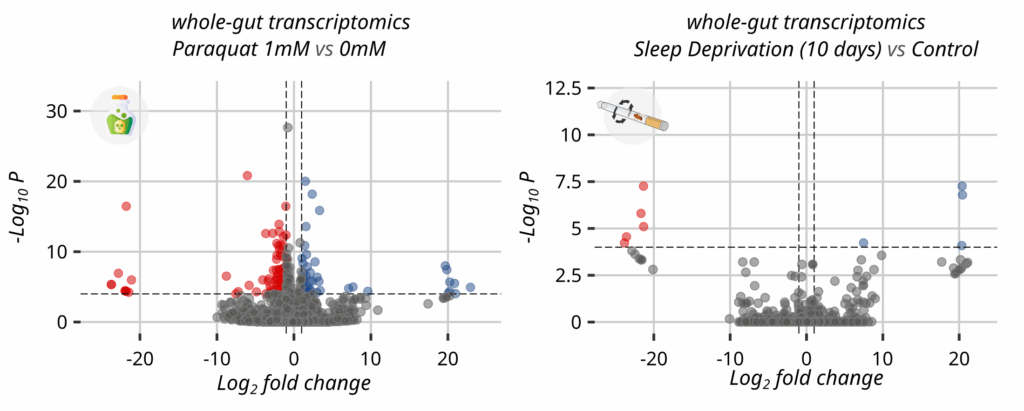
To strengthen the molecular analysis, we also performed transcriptomic of paraquat-induced oxidative stress versus sleep deprivation. The gene expression patterns were completely distinct, with virtually no overlap between pathways activated by oxidative stress and those activated by sleep loss. If sleep deprivation truly caused oxidative damage, we would expect some molecular convergence—but we found none.
The critical insight is that previous sleep deprivation methods inadvertently confounded sleep loss with physical and psychological stress. The ROS accumulation and lethality observed in these studies likely resulted from the stress of the methodology rather than sleep loss itself.
Stress: The Real Culprit
To test this directly, we subjected flies to various forms of stress without depriving them of sleep. The results were striking:
Physical stress: Just 5 minutes of vigorous shaking per day for 4 days caused intestinal ROS accumulation and death
Psychological stress: Flies subjected to social defeat (essentially bullying) by dominant flies showed clear signs of oxidative damage
The same pattern held in mice: Brief restraint stress was enough to trigger intestinal ROS accumulation and damage
These stress paradigms produced the same intestinal phenotype—ROS accumulation, oxidative damage, and ultimately death—that had previously been attributed to sleep loss. But our sleep-deprived flies, kept awake without added stress, showed none of these effects.
The Plot Twist: Sleep Deprivation Creates Vulnerability
Here’s where the story gets interesting. While sleep deprivation alone didn’t kill flies or cause oxidative damage, it did make them more vulnerable to trauma. Sleep-deprived flies were more likely to die when subjected to physical stress, but only under specific conditions.
We subjected flies to two different types of physical force: violent shaking (which constantly changes direction) and centrifugal force (which maintains a steady direction). Both methods applied similar levels of force to the flies, but only the shaking proved lethal. The centrifuge treatment caused no deaths at all. This revealed that it wasn’t the force itself or the procedural stress that was dangerous, but rather the chaotic, multi-directional nature of shaking that caused the trauma.
To understand this better, we examined what happened when we combined sleep deprivation with the shaking treatment. We found that flies deprived of sleep for 24 hours showed dramatically increased mortality when subjected to shaking—but this effect disappeared if we allowed them 6 hours of recovery sleep first. Even more intriguingly, when we tested various genetic mutants with naturally short sleep, we discovered something unexpected: their vulnerability to shaking didn’t correlate with how little they slept. Some short-sleeping mutants were actually more resistant to shaking trauma, while others were more vulnerable. The pattern seemed to depend not on sleep duration, but on the specific neural pathways affected by each mutation.
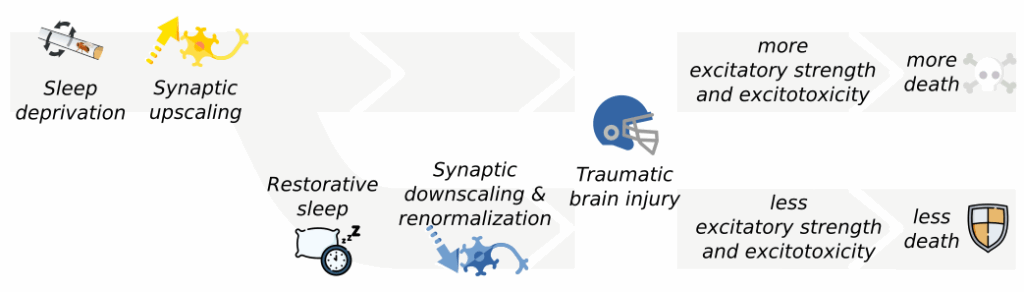
The key turned out to be brain excitability. Sleep deprivation strengthens synapses (the connections between neurons), essentially putting the brain in a hyperactive state. When trauma strikes this “primed” brain, it triggers a cascade of toxic reactions that can prove fatal—exacerbating the violence of a traumatic brain injury. Remarkably, flies with genetic mutations that prevented this synaptic strengthening didn’t show increased vulnerability when sleep-deprived. The problem wasn’t sleep loss itself, but the heightened brain state it created.
What This Means for Humans
This research doesn’t mean you should pull all-nighters without concern. Sleep deprivation in humans causes well-documented problems: impaired cognition, weakened immunity, mood disturbances, and increased accident risk. But these effects might be more about the brain operating in a vulnerable, hyperexcitable state rather than accumulating irreversible damage.
The findings also help explain why stress management is often more effective than simply trying to sleep longer for people with insomnia. Modern sleep medicine increasingly recognizes that stress and sleep problems create vicious cycles—stress disrupts sleep, poor sleep amplifies stress sensitivity, and the cycle continues.
Importantly, while we’ve shown that controlled sleep deprivation doesn’t cause the intestinal ROS accumulation seen in earlier studies, we’re not dismissing the association between sleep loss and gut health. Chronic sleep restriction in real-world scenarios is almost always accompanied by stress, and the combination may indeed lead to oxidative damage. The crucial distinction is that stress, not sleep loss itself, is the primary driver of this damage.
The Bigger Picture
This research represents more than just a correction to sleep science—it’s a reminder of how methodological assumptions can shape entire fields of study. For over a century, the inability to separate sleep loss from stress led researchers down the wrong path.
The Vaccaro study was a major advance in identifying the gut as a critical organ and ROS as a key mechanism in mortality following sleep deprivation paradigms. Our work doesn’t refute those findings—it refines them by demonstrating that the ROS accumulation results from stress inherent in traditional sleep deprivation methods rather than from sleep loss per se.
The real lesson might be that sleep deprivation doesn’t slowly poison us, but rather leaves us vulnerable to life’s inevitable stressors. A sleep-deprived brain isn’t a damaged brain—it’s a primed one, heightened in its responses but fragile when confronted with challenges.
In our stress-filled modern world, perhaps the focus shouldn’t just be on getting eight hours of sleep, but on creating conditions where both stress and sleep can be properly managed together. After all, as this research shows, it might not be the sleep loss that’s the problem—it’s everything else that comes with it.
Links and experimental data
Ethoscope db files for all the behavioural data in the work (TBC)
Metadata, analysis notebooks, confocal images, RNASeq data (Zenodo)
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
What is coccinella?
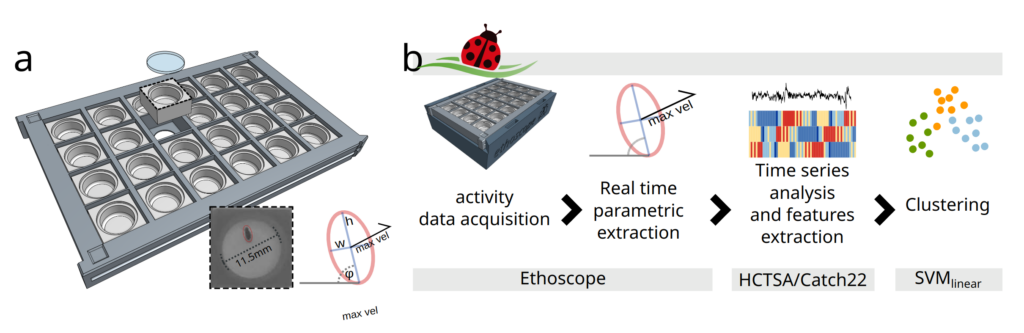
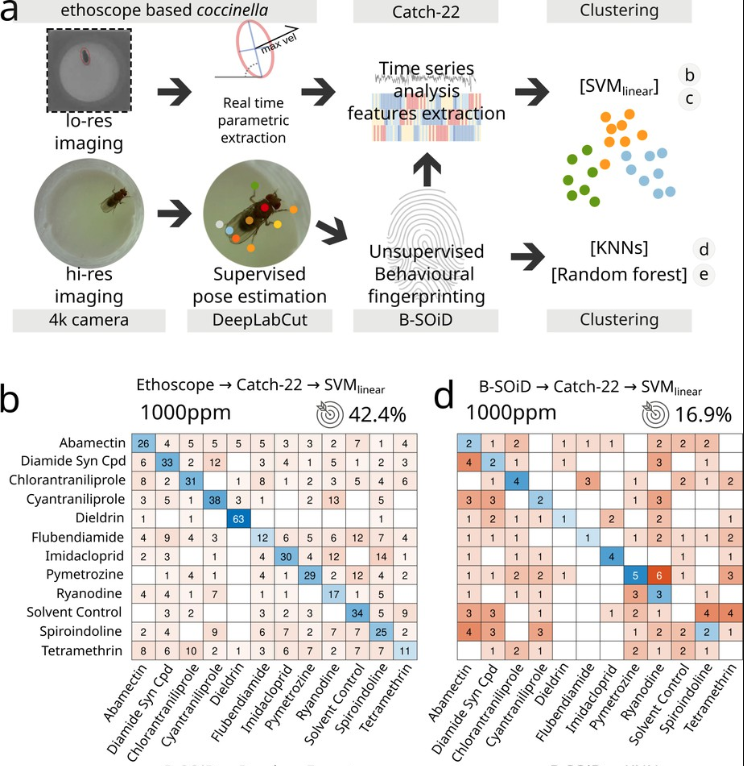
Coccinella is an innovative open-source framework developed for high-throughput behavioral analysis. Leveraging the power of distributed microcomputers, it facilitates real-time tracking of small animals, such as Drosophila melanogaster. Complementing this tracking capability, coccinella employs advanced statistical learning techniques to decipher and categorize observed behaviors. Unlike many high-resolution systems that often require significant resources and may compromise on throughput, coccinella strikes a balance, offering both precision and efficiency. Built upon the foundation of ethoscopes, this platform extracts minimalist yet crucial information from behavioral paradigms. Notably, in comparative studies, coccinella has demonstrated superior performance in recognizing pharmacobehavioral patterns, achieving this at a fraction of the cost of other state-of-the-art systems. This framework promises to complement current ethomics tools by providing a cost-effective, efficient, and precise tool for behavioral research. Coccinella analysis can be done in ethoscopy, a Python framework for analysis of ethoscope data.
How does it work?
Coccinella uses ethoscopes to extract information about the activity of flies in real time. Ethoscopes are machines that use distributed computing via Raspberry PI to detect and interfere with behaviour. Given the off-the-shelf nature of the devices, the all setup is inexpensive and scales up very easily. As term of reference: our lab currently employs about 100 ethoscopes, with a processing power of 20 flies each.
Data about the activity of the animal are then fed to a high-throughput toolbox for time series analysis called HCTSA or Catch22, initially developed at Imperial College London by our colleagues in the Maths Department. The toolbox performs numerous statistical tests aimed at segregating data in an unsupervised way and can therefore be used to cluster together data that the machine recognises as similar. In our case, we tried to identify which drugs have similar mode of action, potentially recognising and assigning the appropriate pharmacological pathways to new, uncharacterized compounds.
We also compared the performance of coccinella to state of the art systems and found that it performs even better!
This is important from the technical point of view but also from the standpoint of neuroscience because it shows that “less is more” when it comes to extracting and recognising behavioural data. In other words, you don’t need to carefully label posture and movement when characterising behaviour: reducing activity to its minimal terms actually works even better!
Joyce, M., Falconio, F.A., Blackhurst, L. et al. Divergent evolution of sleep in Drosophila species. Nat Commun15, 5091 (2024). https://doi.org/10.1038/s41467-024-49501-9
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
Elephants spend up to 18 hours a day eating grass, bushes, roots, shrubs to maintain their appropriate calorie intake. They sleep only 1 or 2 hours a day. Bats, on the other hand, are believed to sleep more than 20 hours a day. Finally, Great Frigatebird. They would normally sleep 9-10 hours a day and you would have hard time trying to get them to sleep less than that. Unless it’s migratory season. In that case, they sleep 40 minutes a day, while they flies for days and days in a row. Evolution is one of the great mysteries of sleep. Why do some animals require 20 hours, while others can cope with 1 or 2? Whatever sleep function is, how can it be accomplished in 10 hours in one season and 40 minutes in another, as it happens in migratory birds?
We won’t really understand what sleep is and what it does if we keep thinking about it in an anthropocentric way. We need to look at it from the evolutionary standpoint and only then we will be able to grasp what its role in nature is. This work marks our first big attempt in this direction. We did not compare sleep between elephants and bats. Too tricky to keep in the test tube and too evolutionary distant. Instead, we used seven species of Drosophila spanning an evolutionary distance of 5-50 Million years and with different ancestral origins and adaptation niches.
In all of them, we measure sleep using a computerised video tracking system based on Raspberry PIs which can be linked to robots to deliver sensory stimuli in real-time, such as puffs of air or automatic rotations of the test tube to keep them awake. We had actually used this device before to explore how fruitflies recognise and respond to salient stimuli during sleep. Here, we combined those with the excellent hidden Markov chain model initially proposed by the Griffith Lab at Brandeis and were able to confirm that different sleep stages as detected by the Markov chain do indeed coincide with different arousabilities. Deep sleeping flies are harder to wake up!
We found that all species sleep in more or less the same way, although for very different lengths of time. In almost all species, sleep is sexually dimorphic: females sleep only at night and males sleep in the afternoon too. Except for D. virilis: a cosmopolitan species believed to have arisen in the Miocene in the deserts of Afghanistan. Interestingly, this is something very recently found in other desert species too. You probably don’t want to be flying around in a desertic afternoon! So, sleep amount is generally conserved and obviously it adapts to species-specific ecological conditions, exactly as for the elephant and the bat. But what about sleep homeostasis? How do these exotic flies react when we try to keep them awake? For this, we turned to our trusty robots and kept flies awake for 24 hours in a row by rotating their little world around every time the fell asleep. A bit like in the Inception movie. Watch the first tube from the left to see the robot in action.
When you deprive an animal of sleep, it tries to recover some of it ASAP. This is a hallmark of sleep homeostasis and what we observed in D. melanogaster, but not in any of the other species! Like the migratory birds, they suddenly seemed OK not sleeping. No signs of tiredness. And even making our robot work for 7 days in a row – 168 hours – did nothing to them! These other species could stay awake just fine and showed no signs of tiredness. Except for melanogaster, which showed a steady increase in sleep pressure. However, at least some species were able to show rebound sleep when we used a different way of keeping them awake: social stress induced by male-male interaction in a laboratory boxing-ring equivalent. Stress can induce rebound sleep in many species, including rodents, and it does so by activating specific brain circuits as our colleagues recently showed.
Surprisingly, male-male interaction did lead to sleep rebound not just in melanogaster but also, simulans, sechelia, yakuba. Still no signs of homeostasis in the remaining three species though! What decides whether an animal will show homestasis? It seems the answer is in their brains. We found that, in general, sleep rebound correlated with an increase in synaptic strength. All the flies that showed rebound also showed a larger amount of a specific synaptic protein. And conversely, when we remove synaptic proteins from specific parts of the brain involved in learning and memory in D. melanogaster we get a similar effect: no tiredness after sleep deprivation.
We also go on and look at the evolution of pharmacology in these species and much more. Have a go at the manuscript yourself. It’s hopefully easy to read for everyone. hat is the take-home message? Well, we try to figure out what all this means in evolutionary terms. We think sleep has different functions in different species (doh!) and some functions therefore evolved for some species but not others. The one common thing all animals have in common is they all sit on the same planet which has been rotating at the same speed for a very long time. We believe this adaptation created sleep in the first place giving animals a chance to optimise their activities to days & nights. Then, other sleep functions kicked in. Some animals need sleep to cope with stress; some others need sleep to learn better; to memorize; to fight bacteria. Who knows how many different functions there are? Some need sleep for multiple reasons at once. This makes sense on multiple levels and can ultimately explain why elephants can do in 1 hour what bats seem to take 20 hours for!
Ethoscope-lab is a pre-baked Docker container featuring an installation of the multi user Jupyter Hub with Python and R kernels, ready to be used with Ethoscopy and Rethomics.
Why using ethoscope-lab?
Let me simply explain how we use it in our lab. We arranged a powerful workstation that acts as lab server and run a dockerized ethoscope-lab on it. The workstation has a local copy of all our ethoscope data (about 8 Terabyte as I type) and ethoscope-lab has local access on those, offering the quickest loading time. Users can then use their computer, or tablet to connect to the workstation and perform data analysis directly from the browser. The setup frees them from working at their desk and allows access to their data from anywhere in the world, guaranteeing at the same time the fastest computational performance even when they work on their laptops. Moreover, the system uses Jupyter notebook as default, meaning each analysis can be nicely annotated and exported to be shared with the world post-publication, along the original raw data.
To give a practical example: this series of repositories on zenodo contains the entire dataset of our latest paper (316Gb) and it’s paired to all the notebooks we used to generate each figure. Readers can download the dataset freely, install ethoscope-lab as docker container on any computer (irrespective of the operating system they adopt) and reproduce all our analyses!
On 29 September 2021 by Giorgio With 0 Comments
- papers
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
One of the most puzzling aspects of sleep is that it cannot happen without depriving us of our full conscious experience. Whatever the function of sleep is, it cannot be achieved without disconnecting our brains from the external world. A full conscious state and sleep are not compatible, it seems, to the point that one of the definitions of consciousness is that “it is all that fades away when we are in dreamless sleep”.
The fact that the brain has to surrender to the tyranny of sleep is also the main reason why scientists believe (in a rather dogmatic fashion) that sleep is “of the brain, by the brain for the brain“. Yet, even during sleep parts of our brains retain some ability to process external information. In the 1960s, Oswald et al formally showed that sleeping humans could wake up in response to some salient stimuli, such as their names being called, but not in response to stimuli of identical strength but no salience, such as other people’s names or their names played in reverse.
This finding has been confirmed and extended over the decades in the scientific literature, providing evidence that it applies to even more complex nuances of saliency, such as an angry tone of voice. The videos below suggest that scientific literature is certainly less comprehensive and (less amusing) than the phenomenon in its entirety.
Pets wake up to food odours and food-related noises.And the human brain is certainly able of very deep sensory processing!
Even though we have numerous scientific and anecdotal evidence that animals and humans can wake up to salient sensory stimuli during sleep, hardly anything is known about the biological underpinning of this phenomenon. And here: enter Drosophila melanogaster! What better animal model than flies to dissect this amazing brain property?
In a paper titled “Sensory processing during sleep in Drosophila melanogaster” published in Nature, we introduce flies as the ideal animal model to dive into the biology of how a brain can simultaneously be asleep and respond to external stimuli.
Postdoc Alice French took the lead on this amazing project to show that even flies can recognise salient stimuli in their sleep and react accordingly, modulating their response based on their internal state. We initially expanded the robotic platform we had previously built in the lab, called ethoscopes, which allows us to monitor and interfere with flies using inexpensive @Raspberry_Pi computers. Alice wanted to build a robotic component able to challenge single flies with specific odour but only while they were asleep, to record whether they would wake up or not. She obviously started with…. LEGO!
In our first prototype, we built a robot able to operate a LEGO valve so to send a puff of air to the sleeping fly. LEGO valves were a good start because we needed 500 of them.
The system worked and we went from those early all-LEGO prototypes (left) to the final 3D printed product (right).
Using this ethoscope module we could challenge sleeping flies with different odours and check whether they would respond differently to some of them. We found they did! Flies would respond to 5% acetic acid for instance, but not to 10% acetic acid. Not only that, the valence of the odour could be modulated by internal states. Flies that had received a little starvation were increasing their response specifically to food-related odours. When we gave alcohol to flies, on the other hand, we found drunk Drosophilae were less responsive to odours in general showing somehow a deeper sleep state.
Now, flies are arguably the best animal model to study circuit neuroscience these days. We have a full connectome of the fly brain and countless genetic tools that allow us to turn neurons on and off. So that is what we did. We started turning neurons on and off in the fly brain, looking for some that would modulate their ability to sense stimuli during sleep. We found them!
We actually found the whole circuit, connecting the “fly nose” all the way to the sleep centers in the brain. And when we used thermogenetics to switch those neurons on or off with infrared radiation, we could interfere with that process and make the flies more or less responsive.
In short, we have shown that flies can recognise and respond to odours during sleep, waking up only to those that they consider salient. We also show that this phenomenon is plastic and modulated by internal states, with animals being more likely to wake to food odours after a little starvation. We also described a blueprint for a neuronal circuit that connects the peripheral olfactory receptor neurons all the way to known sleep-regulating centres in the fly brain. We explore three prototypical gate-points that modulate subconscious processing of olfactory information during sleep: two at the periphery and one in the central brain.
The story is important and of general interest for at least three reasons:
for the groundbreaking implications it has on the consciousness field, introducing flies as a model to study subconscious processing of information, and providing an experimental paradigm that allows to empirically face some key questions of the field;
for the implications it has on the sleep community, describing the neuronal circuit regulating sensory processing during sleep, a neuronal feature that is poorly understood in any other animal model. Our description of the circuit regulating sensory processing during sleep is the most accurate to date and the work also potential future medical significance, for instance in the study of altered states of consciousness, such as coma;
for the implications it has on the larger neuroscience community, describing how a circuit modulates the processing of sensory information to distinguish valence.
Drosophila has been employed to study arousal threshold many times before. There are many studies in which flies can be used to gauge sleep “depth” by using quantitative mechanical stimuli, such as simple vibration or touch. Our study is the first one to study a more puzzling property: how do we recognise qualitative stimuli during sleep? How do we recognise our own name while unconscious?
The video abstract below provides more information on the contents and the implications of the work.
Nat Protoc. 2012 Apr 26;7(5):995-1007.
Video tracking and analysis of sleep in Drosophila melanogaster.
Giorgio F. Gilestro
In the past decade, Drosophila has emerged as an ideal model organism for studying the genetic components of sleep as well as its regulation and functions. In fruit flies, sleep can be conveniently estimated by measuring the locomotor activity of the flies using techniques and instruments adapted from the field of circadian behavior. However, proper analysis of sleep requires degrees of spatial and temporal resolution higher than is needed by circadian scientists, as well as different algorithms and software for data analysis. Here I describe how to perform sleep experiments in flies using techniques and software (pySolo and pySolo-Video) previously developed in my laboratory. I focus on computer-assisted video tracking to monitor fly activity. I explain how to plan a sleep analysis experiment that covers the basic aspects of sleep, how to prepare the necessary equipment and how to analyze the data. By using this protocol, a typical sleep analysis experiment can be completed in 5-7 d.
PLOS Biology, 19 Oct 2017; 15(10): e2003026
Ethoscopes: An Open Platform For High-Throughput Ethomics
Quentin Geissmann, Luis Garcia Rodriguez, Esteban J. Beckwith, Alice S. French, Arian R Jamasb, and Giorgio F Gilestro
We present ethoscopes, machines for high-throughput analysis of behaviour in Drosophila and other animals. Ethoscopes provide a software and hardware solution that is reproducible and easily scalable. They perform, in real-time, tracking and profiling of behaviour using a supervised machine learning algorithm; can deliver behaviourally-triggered stimuli to flies in a feedback-loop mode; are highly customisable and open source. Ethoscopes can be built easily using 3D printing technology and rely on Raspberry Pi microcomputers and Arduino boards to provide affordable and flexible hardware. All software and construction specifications are available at http://lab.gilest.ro/ethoscope.