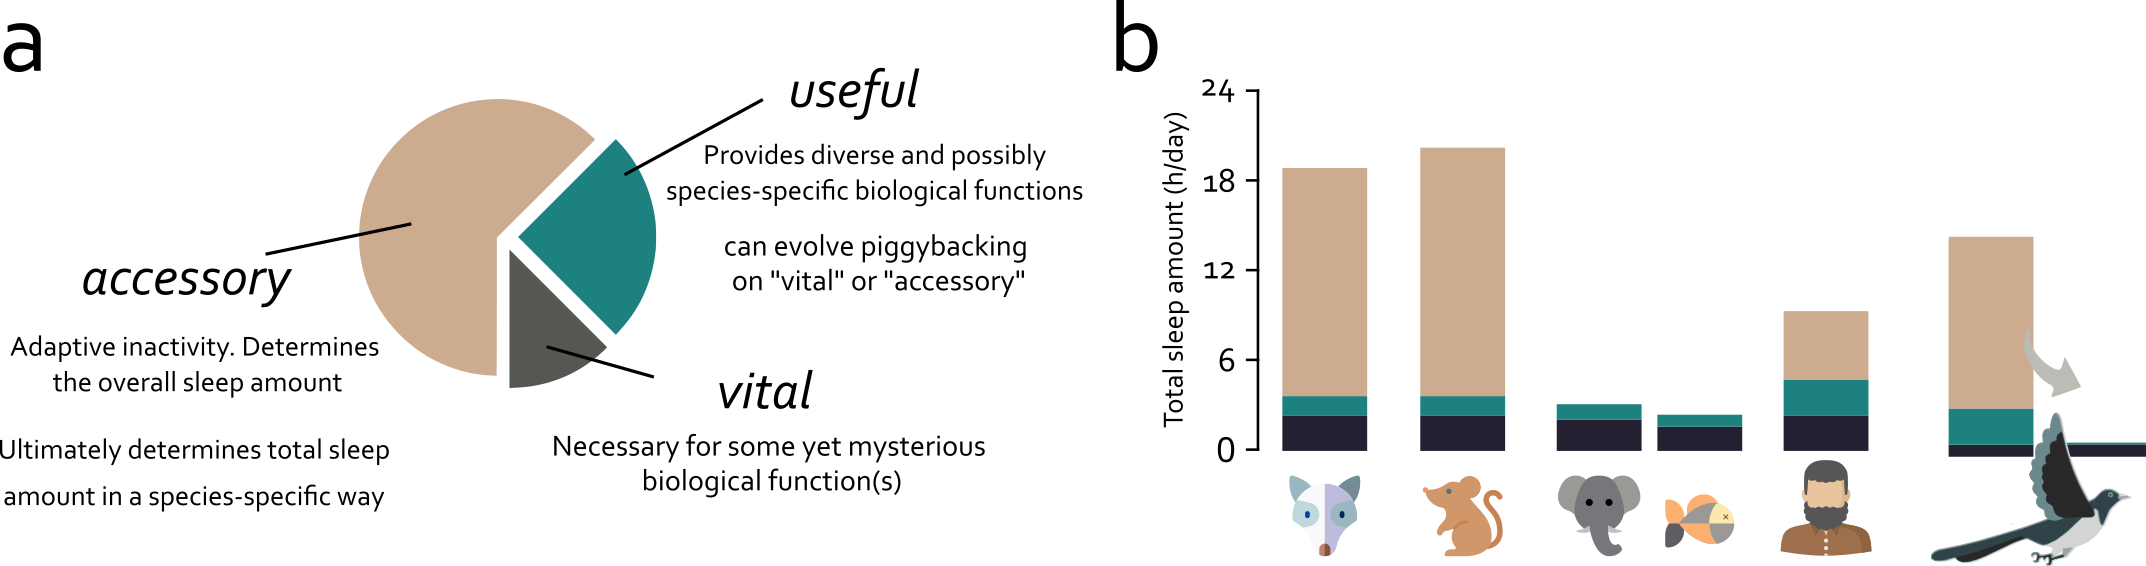On 17 September 2026 by Giorgio With 0 Comments
- papers
Almost every AI model released this year is descended from another one. Some were made by taking a big model and training it a little further on a narrow task. Some were trained on text that an earlier model wrote. Some were built by taking two existing models and averaging the millions of numbers inside them, which sounds like it should not work, and often does. Public repositories, like Hugging Face, now hold millions of these things, and their family trees have already been drawn by people using software written for tracing species.
A group whose members inherit from one another, combine, and pass the result on again is a population, in the sense a biologist means it. Biology has spent a century working out what happens to populations, and what I found is that the theory carries over to machines with its numbers still attached.
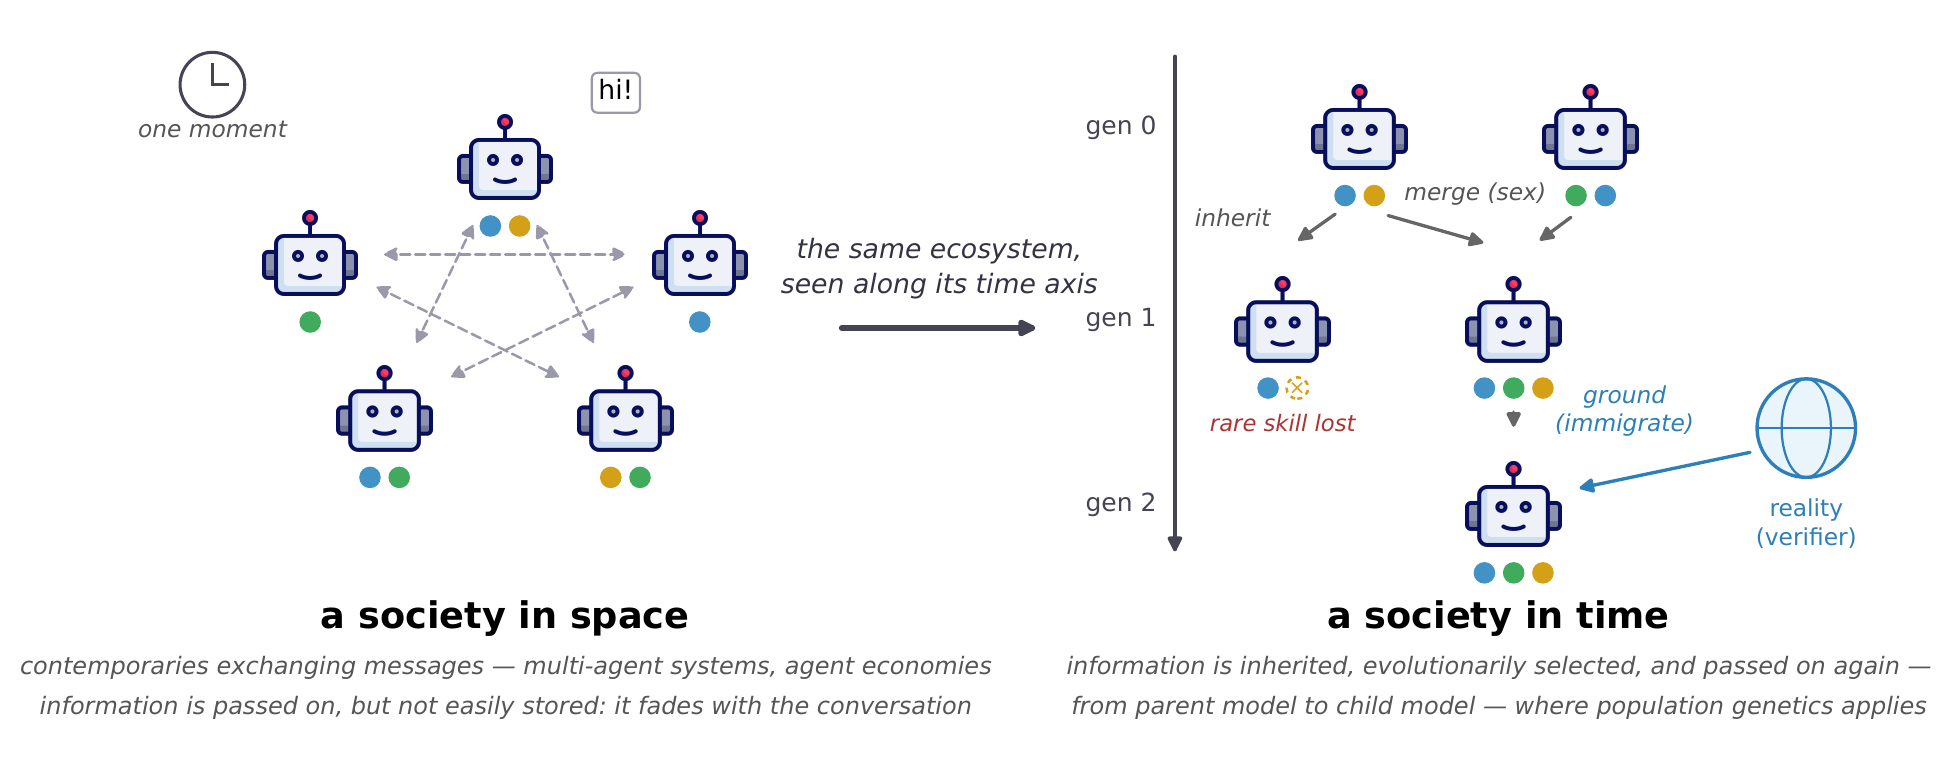
The same ecosystem seen two ways. On the left, models as contemporaries exchanging messages. On the right, the couplings that decide what a lineage keeps: inheritance from parent to child, merging between lineages, and verified real data entering each generation. Population genetics describes the picture on the right.
The rare things go first
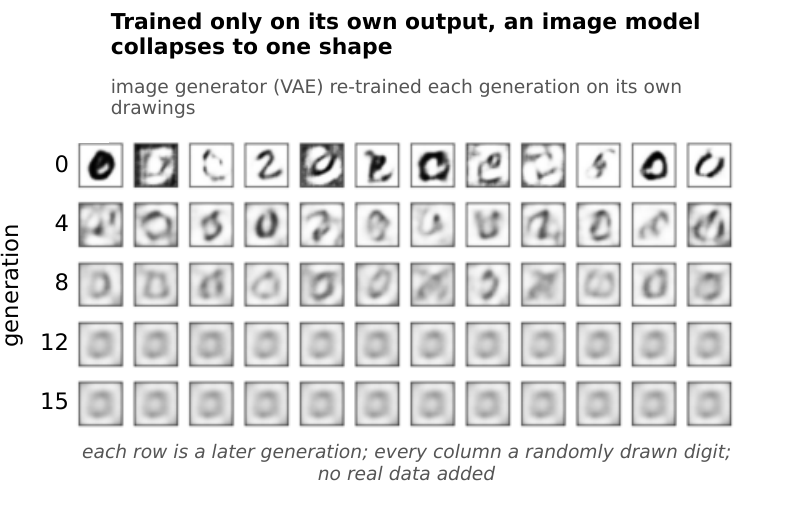
Train a model on the output of the model before it, generation after generation, and it degrades. This is known, and it has a name: model collapse, the term Shumailov and colleagues introduced when they showed it across model families. What is less appreciated is the shape of the damage. Common abilities survive. Rare ones vanish, and they vanish first.
What model collapse actually looks like. Each row is a later generation, trained only on the digits the previous generation drew. Thirty kinds of digit become one shape.
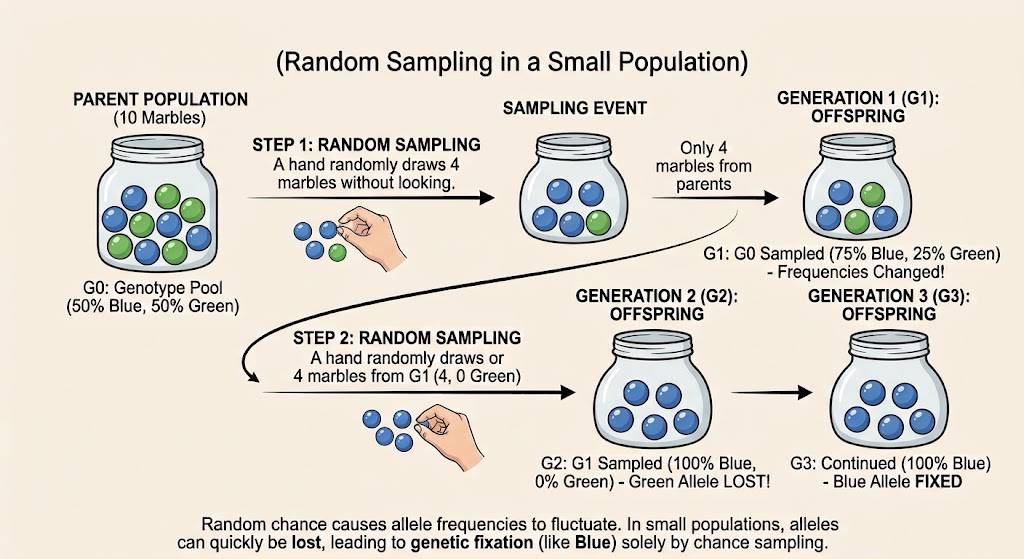
Biologists have known this pattern since the 1930s and it has nothing to do with quality. It is the accident by which rare surnames disappear from small villages: nobody is selecting against them, but each generation is a small sample of the one before, and a name held by two families can be lost by chance in a way that a name held by two hundred cannot. Geneticists call it drift. A model retrained on its own output is running exactly that process, and the maths turns out to be the same equation, not merely a similar one.
How much reality does a model need?
The obvious fix is to keep feeding the thing real human-made data. The question is how much, and here the answer surprised me.
It is not a percentage. It is a count.
What protects a rare ability is the number of real examples of it that reach each generation, and the size of everything else in the training set makes no difference whatsoever. Ten real examples per generation preserve about 95% of the variety, and that is true whether the training set holds two hundred items or two million. Conservation biologists have a rule of thumb for exactly this, worked out for small wild populations: one migrant per generation. One. Not one percent.
The practical version is a budget, and it is a demanding one. To hold on to an ability that shows up in one real example in ten thousand, you need roughly ten thousand real examples every generation, and they have to be examples of that ability. Real data about something else will not do.
A Victorian objection to Darwin, rediscovered by machine learning
Now the part I enjoyed most.
In 1867 an engineer called Fleeming Jenkin published an objection to Darwin that was, at the time, devastating. If children are an average of their parents, he argued, then any rare advantageous trait gets halved at every generation and is watered away to nothing long before natural selection can act on it. Darwin had no good answer. The answer arrived with Mendel: traits do not blend, they pass on whole or not at all. You inherit your grandmother’s eye colour intact, not a smeared average of four grandparents.
Model merging, one of the most popular techniques in AI today, is blending. When you average two models together, an ability held by only one of them gets half the weight, exactly as Jenkin described. I found that machine learning has run into this three separate times, under three different names, without anyone noticing it was the same phenomenon, and that it was a 159-year-old objection to the Origin of Species.
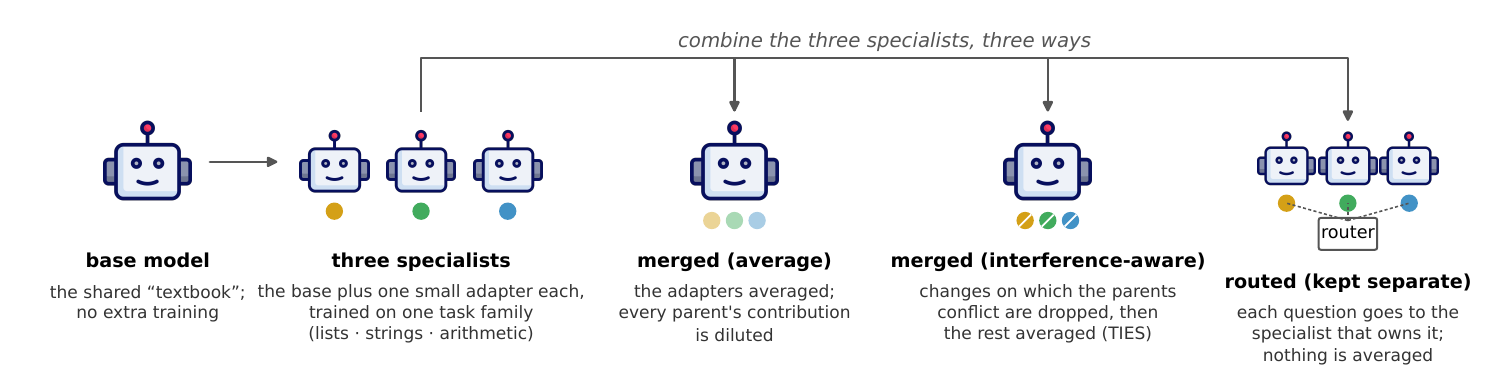
The fix is the one biology arrived at. Stop averaging. Keep the specialists whole and send each question to the one that knows the answer, or generate several candidate offspring and keep whichever tests best. In the experiments, blind averaging on hard tasks did no better than picking the best single specialist. Keeping them separate beat it every time.
Three ways to combine the same three specialists. Averaging fades every parent’s contribution; routing keeps each one whole and sends each question to the specialist that owns it.
When two models can no longer be crossed
A horse and a donkey give you a mule, and the mule is sterile. Somewhere along the way two lineages drift far enough apart that they stop producing viable offspring. That is speciation, and I wanted to know whether it happens to models.
The obvious guess is that models whose internals have drifted far apart will merge badly, and this is what the field currently measures. That guess failed every test I put it to. Two models trained separately on the same skill had almost nothing in common numerically and merged perfectly. Models trained for six times longer than usual merged fine. Language models trained twelve times longer merged better.
What broke merging, every single time, was something more human: the two models had been taught to answer the same question in two different styles. One says “yes” and “no”. The other says “1” and “2”. Both are correct. Neither is compatible with the other, and a merged model has to pick one and be wrong for the other parent forever after.
So the thing that gets inherited in a population of models is not a pile of numbers. It is a convention, a way of answering a kind of question. Most numerical differences between two models are harmless, in much the way that most of the differences between any two human genomes are harmless.
That gives a cheap test, and it works. Before merging two models, ask them both the same set of questions and count how often they disagree. That count predicted how much damage the merge would do. The standard measure, distance between their internals, predicted nothing at all.
A small society of models, over six generations
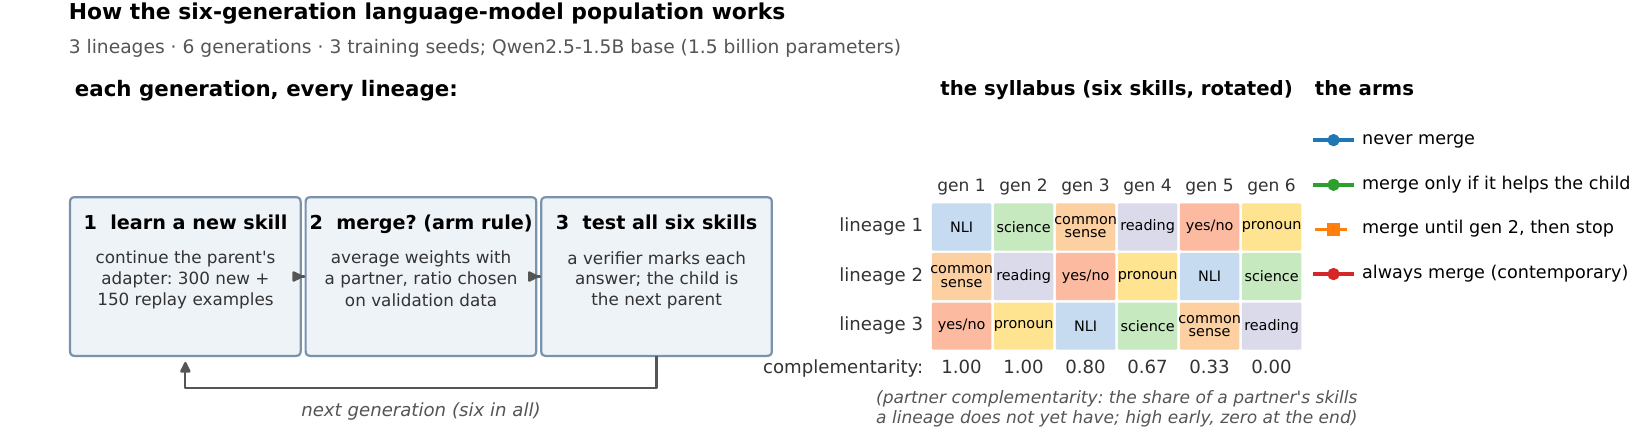
Finally I built a little society: three lineages of language models, each learning a new skill every generation for six generations, each able to merge with the others.
The set-up. Three lineages take the same six skills in a different order, so early on a partner always knows something you do not, and by the end it knows nothing you do not.
Lineages forced to merge every generation did well for three generations and then collapsed. Lineages allowed to refuse a merge (by checking whether the merged offspring was better than the unchanged parent, and keeping whichever won) never collapsed at all.
And the strangest result: merging a model with its own ancestor from three generations back was safer than merging it with a contemporary, in every single run. An ancestor lacks everything you have learned since, so it has something to offer, but it shares every convention you hold, so it cannot contradict you. Biologists have a name for a population that can breed with its own stored past. They call it a seed bank, and it is what a sediment full of dormant seeds does for a plant population.
Why this matters
If you train on synthetic data, budget in counts and not percentages. Almost every published guideline is stated as a fraction of the training set, and the fraction is the wrong unit. The same arithmetic turns up in work on data poisoning, where a near-constant number of documents does the job whatever the size of the model. It also means that the bigger your training set gets, the smaller the percentage you need, which is good news nobody is currently claiming.
If you merge models, averaging is the wrong default. It is the cheapest option and it destroys the specialist abilities you merged in order to keep.
Incompatibility is measurable in advance, and cheaply. Asking two models the same questions costs almost nothing compared with performing a merge and evaluating the wreckage.
And a warning about scale. These models are increasingly trained, evaluated and selected by other models. A population that is scored on how well it agrees with itself, rather than against anything real, converges confidently on a wrong answer. That is not speculation, it is what happened in my simulations whenever I removed the external check. Reality has to keep the right to say no.
Links and further material
The preprint, the code, every configuration file and every random seed are public. The entire study re-runs from one script.
On 19 August 2026 by Giorgio With 0 Comments
- papers
Sleep is universal, it is defended whenever you take it away, and it looks expensive. For half a century those three facts have been read as a single message: sleep must be doing something vital, and we have simply not worked out what yet.
The search has not converged. It has produced a dozen candidate functions (synaptic downscaling, metabolite clearance, memory consolidation, immune support, energy conservation, and more), each defensible in the setting where it was found, none commanding general assent. Fifty years in, that is not what a field looks like when it is closing on an answer.
No two animals sleep alike
There is a fourth fact, and it sits badly with the other three. Animals sleep in very different ways and for very different amounts of time, from around two hours a day in an elephant to twenty in a little brown bat, and the correlates proposed for that range (body mass, diet, position in the food chain) account for only a modest part of it. A cellular transaction that every animal must complete every day, on pain of death, should not vary tenfold in how long it takes.
The variation within a single animal is more awkward still. In some songbirds sleep occupies sixteen hours or more of a winter day and then collapses to minutes a day through migration and the breeding season, for weeks on end, without the rebound that a debt model would demand. Frigatebirds do something comparable over the ocean, sleeping well under an hour a day for a week at a time and behaving normally when they make landfall. In biology, this kind of variability is rarely noise to be averaged away. It is usually the most informative thing on the table, and here it is telling us that most of sleep is negotiable.
So what is it that stretches, and what, if anything, does not?
Fitness, not function
We ask what the function of sleep is, and the trouble is in the definite article. It presupposes that there is one function, that it is the same in a jellyfish and in a human, and that whatever it turns out to be, it justifies spending a third of a life insensible to the world.
Evolution does not optimise function. It optimises fitness. Ask instead what fitness sleep confers, and to whom, and the expectation of a single answer disappears. Different advantages can accrue to different lineages, at different times, layered on top of one another.
What sleep costs
The vocabulary for a quantity that stretches under pressure already exists, and it belongs to economics rather than to biology. In 1890 Alfred Marshall introduced the price elasticity of demand, a measure of how sharply demand for a good falls as the good becomes more expensive. Life-saving medicine is inelastic, because people buy it at almost any price. Luxuries are elastic, and demand for them collapses as soon as the price goes up.
For sleep, the price is everything the animal gives up by being asleep (food not found, mates not courted, territory not defended, predators not watched for), and that price is not a constant. It is set by ecology and it moves with the season. To a songbird in a safe winter roost, with nothing to be gained from being awake in the dark, sleep is close to free. To the same bird crossing the Sahara in spring it is ruinously expensive, and the bird behaves exactly as a buyer facing a sudden price rise. It stops buying.
That is where this framework starts. Which parts of sleep behave like the medicine, and which behave like the luxury?
Three components, one state
In a new preprint I set out what I call the sleep elasticity hypothesis.
An accessory component came first, an ecological buffer that keeps an animal safely and economically inactive through the hours when activity would not repay itself. It discharges no cellular transaction. It has no biochemical function at all, only ecological value, and in most species it is the largest part of the night.
Onto that pre-existing state, individual lineages have since loaded useful processes, memory consolidation in some, immune or metabolic work in others. These are exaptations, recruited onto something that was already there for other reasons. What a species does with its sleep is therefore a fact about the species, and not about sleep.
Whether a third, genuinely vital component exists is a question I hold open rather than answer. If it turns out to be empty, the framework stands with two layers.
Sleep as three superimposed components of distinct evolutionary origin: the accessory buffer of adaptive inactivity, the useful and largely lineage-specific processes exapted onto it, and the vital residue held open as a hypothesis.
The three components differ in exactly the way the economics anticipates. The accessory component is highly elastic, and most of the variation we see between species, and across the seasons of a single life, is variation in it. The useful component is less elastic, in proportion to how heavily a given lineage has come to lean on what it does. Whatever remains, if anything remains, should not move at all.
Why this matters
It explains why the field is stuck. If sleep is a mixture rather than a thing, then every study measuring “sleep” has been measuring a different blend of three components, and the dozen incompatible functions in the literature are exactly what you would expect to find. The contradictions stop being a scandal and start being data.
It makes total sleep duration close to meaningless. Hours on the clock are a compound of amount set by ecology and opportunity, timing by the circadian system, depth by whatever physiological work is being done, and a residue that bounds any indispensable core. Comparing species by how long they sleep, or people by whether they manage eight hours, is comparing sums of quantities that are not the same across the things being compared.
It turns the field’s most embarrassing observations into predictions. The migrating bird that sheds sleep for weeks and never repays it, the cavefish that has lost most of its sleep but kept the homeostat that would defend it, the fur seal that abandons one sleep state at sea while still defending the other: these are anomalies only if sleep is one indispensable thing. Under a layered account they are the expected result of different lineages carrying different loads.
It tells experimentalists what to measure instead. Depth read as arousal threshold, rather than as slow-wave power, is the most promising route to pulling the three components apart. Slow waves are a mammalian signature. Arousal threshold can be measured in anything that behaves, which is what a comparative account of sleep actually needs.
What would sink it
I have tried to state this so it can lose. The paper sets out each claim with the evidence for it, the leading alternative reading, the confidence it warrants, and the observation that would decide it.
The honest weakness is measurement. Nobody can currently decompose an animal’s sleep into accessory, useful and vital parts, and devising a way to do it is the most important experimental challenge the framework sets. Until then the proportions I draw remain a hypothesis, not a result.
A reader who expects a vital core to be found eventually is not refuting this. They are proposing a value for one of its terms.
The elastic, tripartite model was first sketched in 2018 and has been under continuous development since, improved beyond recognition by everyone in my laboratory and by the many colleagues who argued with it at meetings and in seminars over the years. I talked about some of these ideas on multiple podcasts and interviews. Below, the Max Planck Florida’s Neurotransmissions podcast, in an episode titled “Could Sleep be Nature’s Time-out?”.
On 4 February 2026 by Giorgio With 0 Comments
- papers
Updated September 2026: this post was rewritten to follow the current version of the preprint.
In Berlin, around 1904, a horse called Hans drew crowds by tapping out the answers to arithmetic questions with his hoof. Experts examined him and found no trickery. It took a young psychologist to work out what was really happening: Hans was watching the people asking the questions. As his hoof approached the right number, they relaxed very slightly, without realising it, and Hans stopped. When the questioner didn’t know the answer, or stood out of sight, Hans failed. He was doing something clever, but not arithmetic.
Now a second story. Over the last century, crows in New Caledonia were seen making hooked tools from twigs, bending wire into hooks in the laboratory to fish out food, and using one tool to fetch another. Each time, sceptics had a simpler explanation ready: instinct, trial and error, habit. It took decades before scientists accepted that crows really can reason about cause and effect.
These stories are usually told as opposites. In the first, people saw a mind that wasn’t there; in the second, they refused to see one that was. My argument is that they are the same mistake made in opposite directions. In both cases, people decided what they were looking at before weighing the evidence. Hans’s audience saw a performance and assumed a mind behind it, without asking how the taps were produced. The crows’ sceptics knew they were “only birds” and never let the performance count.
The second mistake is older than science. In 1773 Phillis Wheatley, an enslaved young woman in Boston, published a book of remarkable poems. Many refused to believe she had written them. Thomas Jefferson admitted the poems were competent but insisted that their author could not be a poet. The work was accepted; the ability it showed was denied, because of who she was. The same move is being made today about artificial intelligence: yes, the system solved the problem, but it didn’t really reason, it only imitated reasoning.
The first mistake has a name, the Clever Hans effect. The second doesn’t, so I call it the mimicry trap: the behaviour is accepted, but relabelled as mere mimicry, so that a verdict decided in advance survives whatever the evidence shows. Today’s AI chatbots are the first case in which both mistakes are being made at once, and on a huge scale, by the public and by experts alike.
Two kinds of mind
When we judge whether something has a mind, we are really asking two questions. Can it think? And can it feel? In every animal we have ever met, the two go together: creatures that seem cleverer also seem to feel more. So we have learned to treat one as a sign of the other. AI systems are the first case in which the two come apart. They are getting better and better at tasks that look like thinking, while whether they feel anything remains a completely open question. Our old habits of judgement, built on animals, don’t work here.
Turing’s test, updated
In 1950 the mathematician Alan Turing proposed a famous test: if a machine can hold a conversation that you can’t tell apart from a human’s, you should credit it with thinking. Turing judged by behaviour alone, which made sense at the time, because nobody knew what a thinking machine would look like inside.
Today we can look inside, at least partly, and that changes things. My proposal is to treat Turing’s test as a piece of reasoning under uncertainty, the kind a doctor uses. A doctor who sees a symptom asks two questions: how well does this symptom fit the disease? And how likely was the disease in this patient before I saw the symptom? Both matter. For AI, the symptom is the behaviour, and the “before” is what we know about how the system was built. Finding something clever inside (say, a hidden map of a board game that the system was never shown) should raise our confidence. Finding a trick inside (a list of memorised answers) should lower it.
Both mistakes come from refusing to let the evidence move that starting point. The Clever Hans mistake sets it at “obviously intelligent” because the system looks and sounds like someone, and never checks how it works. The mimicry trap sets it at “cannot possibly be intelligent” because of what the system is made of, and nothing it does can change that.
A good test for yourself: would you judge the system differently if exactly the same machine, doing exactly the same things, had arrived from outer space and nobody knew who built it? If so, it is your expectation doing the judging, not the evidence.
What would change your mind?
Imagine AI keeps improving the way it has in the last five years. At what point would a sceptic admit that what they are seeing is no longer mimicry? And the enthusiast owes the mirror answer: what would you have to discover about how the machine works to change your mind?
A good answer has three properties. It names something you could actually observe and check (“genuine understanding” doesn’t count, because nobody can check for it). It is fair: the same evidence would count if a person or an animal produced it. And it is stated in advance, not invented after the previous test has been passed.
This doesn’t say who is right. Many sceptics give perfectly good answers to the question, and some enthusiasts give none. What it rules out is a position that nothing could ever change.
The full preprint is on PhilSci-Archive. What I ask of critics is that they say, in advance, what evidence would change their mind. If the answer is “nothing could”, we are no longer having a scientific conversation.
For over 125 years, scientists have believed that sleep deprivation is lethal. This idea traces back to 1894, when Russian researcher Maria Manaseina made a shocking discovery: puppies forced to stay awake died within just 4-5 days. She declared that “complete absence of sleep is much more fatal for animals than the absolute absence of food”—a statement that has echoed through scientific literature ever since.
But what if we’ve been wrong this entire time?
The problem with sleep deprivation research has always been methodological. How do you keep an animal awake without stressing it? Early researchers resorted to increasingly creative—and harsh—methods: constant poking, forced walking, loud noises, even electric shocks.
Rats running a on a treadmill – if they fall asleep or stop, they hit the back of the treadmill and get an electric shock. A stressful system used for sleep deprivation.
Another system commonly used to keep flies awake: flies experience periodic “earthquakes”, every few minutes. This happens independently of the behavioural state of the animal and it is likely to introduce stress, physical trauma, and interferes with feeding.
When animals died, scientists assumed it was from lack of sleep. But even pioneering sleep researcher Nathaniel Kleitman worried in 1928 that he couldn’t tell “to what extent the effects were due to lack of sleep, and to what extent to muscular fatigue.” This confusion persisted for decades. Even the famous experiments by Allan Rechtschaffen in the 1980s—considered the gold standard of sleep deprivation research—used a method that constantly disturbed rats on a slowly rotating disk. When the rats died after 2-3 weeks, everyone assumed sleep loss was the culprit.
The ROS Revolution: A Breakthrough Discovery
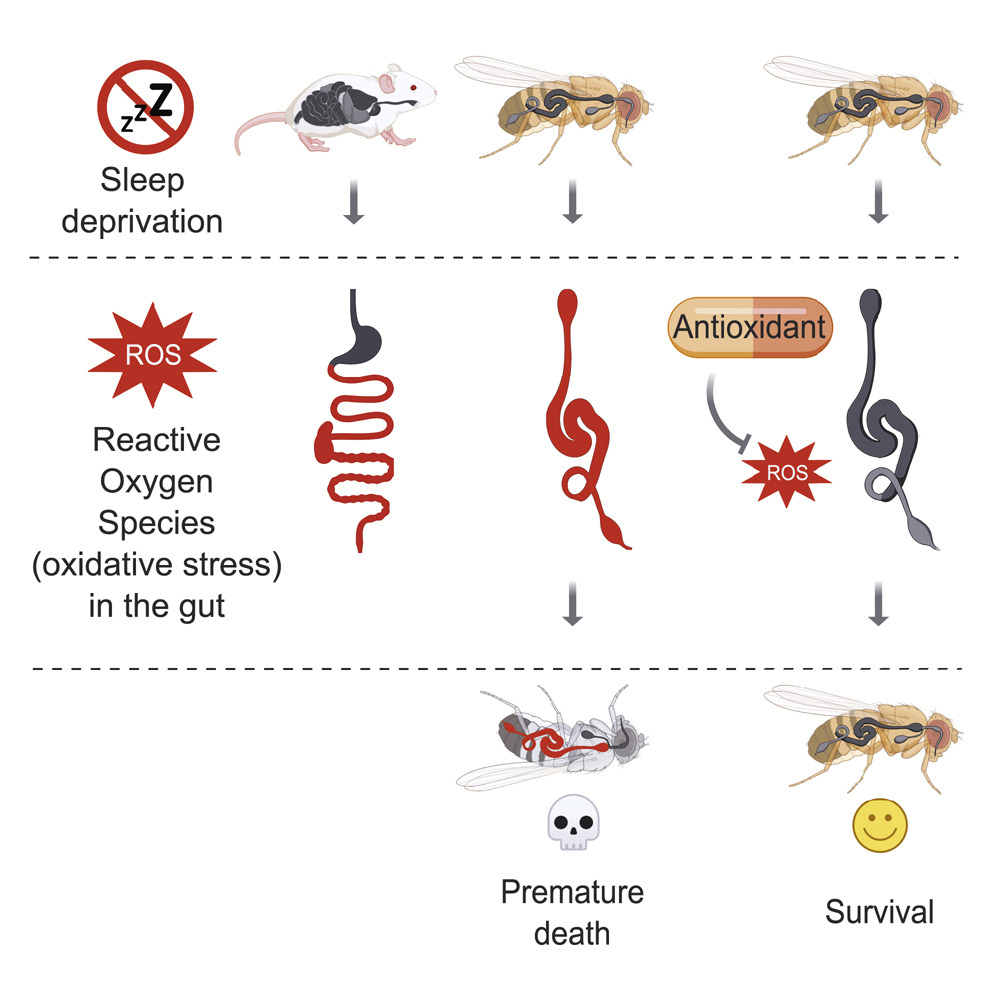
In 2020, a landmark study by Vaccaro and colleagues at Harvard Medical School made what seemed like a definitive discovery about why sleep deprivation kills. Working with both flies and mice, they reported that severe sleep deprivation led to the accumulation of reactive oxygen species (ROS)—highly reactive molecules that can damage cells—specifically in the gut. The findings were compelling: intestinal tissues showed widespread cellular damage, including DNA damage, stress granules, and markers of cell death. When they prevented ROS accumulation using antioxidant compounds or by expressing antioxidant enzymes specifically in the gut, sleep-deprived flies could survive with little to no sleep. The conclusion seemed clear: sleep deprivation kills by causing oxidative damage in the gut.
This discovery was revolutionary because it provided a specific, mechanistic explanation for lethality. It wasn’t just that animals were tired or stressed—there was measurable, progressive damage to a specific organ system. The gut, with its high metabolic activity and regenerative capacity, appeared to be the Achilles heel during prolonged wakefulness.
A Gentler Approach Reveals a Different Truth
Enter the ethoscope: a clever device that uses real-time video tracking to monitor individual fruit flies. Unlike previous methods that constantly harass animals, the ethoscope only intervenes when it detects that a fly is actually sleeping—giving it a gentle nudge to wake up, then leaving it alone during active periods.
Using this stress-controlled approach, we had already found something remarkable back in 2019: flies could be kept awake throughout their lives without dying!
This raised an intriguing question: if Vaccaro’s team found that sleep deprivation caused lethal ROS accumulation in the gut, why were our flies surviving indefinitely? We hypothesized that our gentler, ethoscope-based sleep deprivation method might not induce the same intestinal oxidative damage.
Testing the ROS Hypothesis
To test this directly, we subjected flies to 10 days of continuous sleep deprivation using the ethoscope and examined their intestinal tissues using the same fluorescent probes used by Vaccaro and colleagues—DHE for superoxide detection and H2DCF for hydrogen peroxide detection. The results were striking: we found no ROS accumulation whatsoever.
But we needed to rule out confounding factors. Perhaps dietary antioxidants or the gut microbiome were masking ROS accumulation by scavenging reactive oxygen species before we could detect them? We systematically eliminated these possibilities:
We maintained flies on minimal diet consisting only of 5% sucrose in agar, lacking the complex nutrients and natural antioxidants in standard laboratory food—still no ROS.
We raised axenic flies completely free of microorganisms from embryonic development through adulthood—still no ROS accumulation following sleep deprivation.
We even performed sleep deprivation at higher temperatures (29°C) to accelerate metabolic rate—still no detectable ROS.
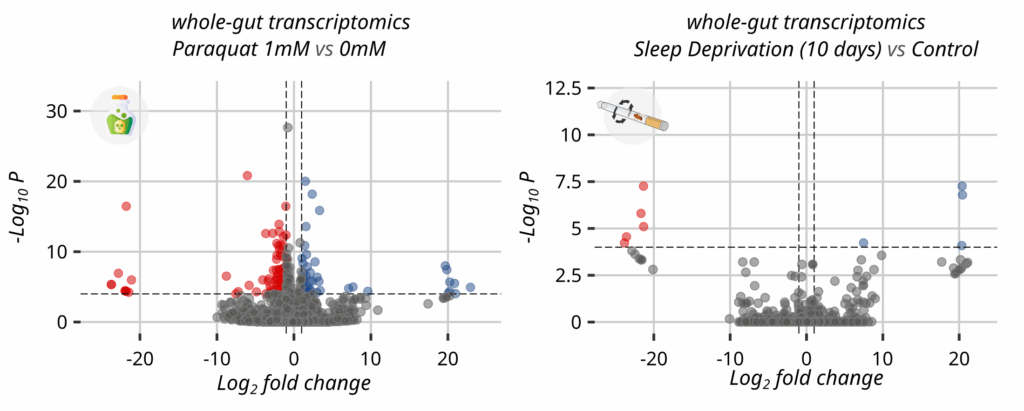
To validate our detection methods, we exposed flies to paraquat, a potent toxin that generates ROS. As expected, even low doses of paraquat produced readily detectable ROS accumulation in the gut. Surprisingly, adding 10 days of sleep deprivation to paraquat treatment produced no additional effect—sleep-deprived animals showed no increase in ROS levels compared to rested controls receiving the same paraquat dose, and no change in survival.
The conclusion was inescapable: ethoscope-based sleep deprivation, even when sustained for 10 days, does not cause intestinal ROS accumulation or oxidative damage.
To strengthen the molecular analysis, we also performed transcriptomic of paraquat-induced oxidative stress versus sleep deprivation. The gene expression patterns were completely distinct, with virtually no overlap between pathways activated by oxidative stress and those activated by sleep loss. If sleep deprivation truly caused oxidative damage, we would expect some molecular convergence—but we found none.
The critical insight is that previous sleep deprivation methods inadvertently confounded sleep loss with physical and psychological stress. The ROS accumulation and lethality observed in these studies likely resulted from the stress of the methodology rather than sleep loss itself.
Stress: The Real Culprit
To test this directly, we subjected flies to various forms of stress without depriving them of sleep. The results were striking:
Physical stress: Just 5 minutes of vigorous shaking per day for 4 days caused intestinal ROS accumulation and death
Psychological stress: Flies subjected to social defeat (essentially bullying) by dominant flies showed clear signs of oxidative damage
The same pattern held in mice: Brief restraint stress was enough to trigger intestinal ROS accumulation and damage
These stress paradigms produced the same intestinal phenotype—ROS accumulation, oxidative damage, and ultimately death—that had previously been attributed to sleep loss. But our sleep-deprived flies, kept awake without added stress, showed none of these effects.
The Plot Twist: Sleep Deprivation Creates Vulnerability
Here’s where the story gets interesting. While sleep deprivation alone didn’t kill flies or cause oxidative damage, it did make them more vulnerable to trauma. Sleep-deprived flies were more likely to die when subjected to physical stress, but only under specific conditions.
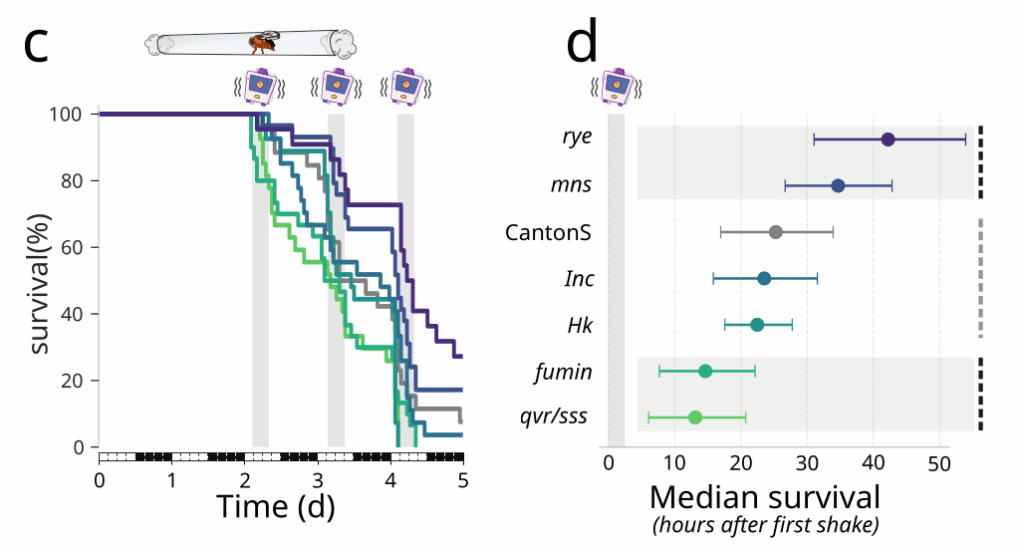
We subjected flies to two different types of physical force: violent shaking (which constantly changes direction) and centrifugal force (which maintains a steady direction). Both methods applied similar levels of force to the flies, but only the shaking proved lethal. The centrifuge treatment caused no deaths at all. This revealed that it wasn’t the force itself or the procedural stress that was dangerous, but rather the chaotic, multi-directional nature of shaking that caused the trauma.
To understand this better, we examined what happened when we combined sleep deprivation with the shaking treatment. We found that flies deprived of sleep for 24 hours showed dramatically increased mortality when subjected to shaking—but this effect disappeared if we allowed them 6 hours of recovery sleep first. Even more intriguingly, when we tested various genetic mutants with naturally short sleep, we discovered something unexpected: their vulnerability to shaking didn’t correlate with how little they slept. Some short-sleeping mutants were actually more resistant to shaking trauma, while others were more vulnerable. The pattern seemed to depend not on sleep duration, but on the specific neural pathways affected by each mutation.
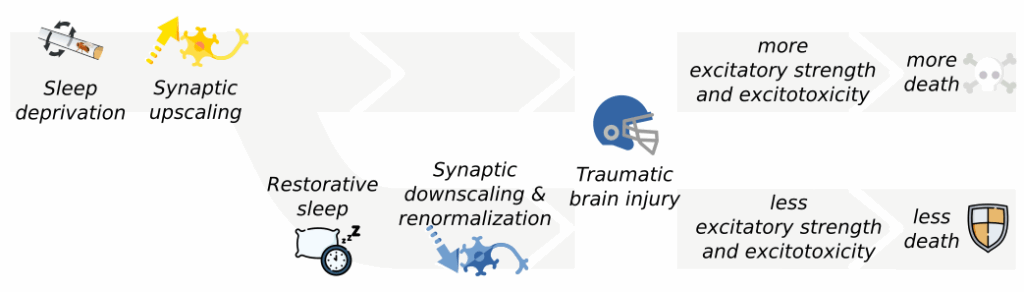
The key turned out to be brain excitability. Sleep deprivation strengthens synapses (the connections between neurons), essentially putting the brain in a hyperactive state. When trauma strikes this “primed” brain, it triggers a cascade of toxic reactions that can prove fatal—exacerbating the violence of a traumatic brain injury. Remarkably, flies with genetic mutations that prevented this synaptic strengthening didn’t show increased vulnerability when sleep-deprived. The problem wasn’t sleep loss itself, but the heightened brain state it created.
What This Means for Humans
This research doesn’t mean you should pull all-nighters without concern. Sleep deprivation in humans causes well-documented problems: impaired cognition, weakened immunity, mood disturbances, and increased accident risk. But these effects might be more about the brain operating in a vulnerable, hyperexcitable state rather than accumulating irreversible damage.
The findings also help explain why stress management is often more effective than simply trying to sleep longer for people with insomnia. Modern sleep medicine increasingly recognizes that stress and sleep problems create vicious cycles—stress disrupts sleep, poor sleep amplifies stress sensitivity, and the cycle continues.
Importantly, while we’ve shown that controlled sleep deprivation doesn’t cause the intestinal ROS accumulation seen in earlier studies, we’re not dismissing the association between sleep loss and gut health. Chronic sleep restriction in real-world scenarios is almost always accompanied by stress, and the combination may indeed lead to oxidative damage. The crucial distinction is that stress, not sleep loss itself, is the primary driver of this damage.
The Bigger Picture
This research represents more than just a correction to sleep science—it’s a reminder of how methodological assumptions can shape entire fields of study. For over a century, the inability to separate sleep loss from stress led researchers down the wrong path.
The Vaccaro study was a major advance in identifying the gut as a critical organ and ROS as a key mechanism in mortality following sleep deprivation paradigms. Our work doesn’t refute those findings—it refines them by demonstrating that the ROS accumulation results from stress inherent in traditional sleep deprivation methods rather than from sleep loss per se.
The real lesson might be that sleep deprivation doesn’t slowly poison us, but rather leaves us vulnerable to life’s inevitable stressors. A sleep-deprived brain isn’t a damaged brain—it’s a primed one, heightened in its responses but fragile when confronted with challenges.
In our stress-filled modern world, perhaps the focus shouldn’t just be on getting eight hours of sleep, but on creating conditions where both stress and sleep can be properly managed together. After all, as this research shows, it might not be the sleep loss that’s the problem—it’s everything else that comes with it.
Links and experimental data
Ethoscope db files for all the behavioural data in the work (TBC)
Metadata, analysis notebooks, confocal images, RNASeq data (Zenodo)
Below is the English translation of a seminal paper by Marie de Manacéïne, dated 1880. The original writing, in French, appeared as “Quelques observations sur l’influence de l’insomnie absolue. Arch. ital. de Biol., p. 322, 1894, aussi Congrès de Rome, vol II, p 174” and it is available here as PDF. A biography of Marie de Manacéïne can be found here. Translation by Giorgio Gilestro.
While observations on normal (2) and artificial sleep are becoming increasingly numerous, absolute insomnia or complete sleep deprivation has not yet been the subject of experimental research. However, to fully understand the role of sleep in organic life, it would also be necessary to know the influence of complete sleep deprivation. It is known that in China and in antiquity, among the different types of torture, there was death caused by sleep deprivation, that is to say, the condemned was kept from sleeping and was awakened each time he began to fall asleep. Facts of this kind clearly demonstrate that sleep deprivation produces one of the most harmful influences.
On the other hand, observations collected in clinics and in private medical practice have shown that most patients suffering from insomnia do not present a total lack of sleep, but that they only have very fleeting and short sleep (Hammond), and that this insufficient sleep is already capable of seriously disturbing the general health of people who are subject to it. Dr. Renaudin (3) observed that this partial insomnia is already sufficient to cause the development of more or less serious disorders of psychic life. Complete or absolute insomnia is extremely rare, and according to the observations of Prof. Hammond (4), it quickly ends in death; in fact, in an experiment where he observed absolute insomnia for 9 days, death occurred precisely during the 9th day.
All these facts demonstrate how important the experimental study of the influence of a complete lack of sleep must be, and this is what decided me to attempt an experimental study of absolute insomnia. My experiments were conducted on young dogs aged two, three and four months. All these dogs were still mainly feeding on their mother’s milk, and this circumstance was very useful for experiments of this nature, as the presence of their mother was much more effective than all other manipulations in keeping them awake. The number of these experiments was very limited, as they are extremely painful for the experimenter; indeed, he must constantly pay the utmost attention to the animals, which have a tendency to fall asleep at any moment and even in the most uncomfortable positions. I experimented only on ten young dogs; but, as the results obtained were absolutely identical in all cases, I thought that these experiments could suffice and that it was unnecessary to make more of these poor beasts perish.
The experiments carried out on young dogs have shown that the complete absence of sleep is much more fatal for animals than the absolute absence of food. One can hope to save animals that have undergone complete starvation for 20-25 days and even for a longer time, one can save them even after they have lost more than 50% of their weight, while in cases of absolute insomnia the animals were irreparably lost, even after sleep deprivation of 120 to 96 hours. No matter how much they were warmed up and artificially fed all the time and given the full possibility to sleep comfortably – they would still die. Out of ten dogs, I left four without sleep until death, while for the other six I tried to save them after insomnia of 120-96 hours. The first four dogs died after complete sleep deprivation for 92 to 143 hours. Older dogs endured the lack of sleep longer than younger dogs, – which is quite natural, because everyone knows that the younger an organism is, the more it needs sleep. The temperature of young dogs deprived of sleep begins to drop in the second 24 hours of insomnia, where it shows a decrease of 0.5 to 0.9 C; then the decrease becomes more and more rapid, and towards the final hours of life, the animals’ temperature is already 4° to 5° and even 5.8°C below normal. With the first drops in temperature, we notice very pronounced changes in reflex movements, which become slower and weaker and, at the same time, show a certain periodicity, appearing more or less absent, sometimes on one side of the body, sometimes on the other. The reaction of the pupils to light and darkness shows the same changes and the same periodicity as other reflex muscle movements. We sometimes notice, in sleep-deprived dogs, a pronounced inequality of the pupils. The number of red blood cells shows marked changes: after 48, 55, 96 and 110 hours of insomnia, the number of red blood cells was found to be reduced from 5,000,000 to 3,000,000 and even to 2,000,000 in a cubic millimeter.
Towards the end of life, that is, during the last 24 or 36 hours, we observe an apparent increase in red blood cells and hemoglobin; but this apparent increase depends on the fact that the animals refuse to eat or drink during the last 48 hours, and as their kidneys continue to function, they lose more and more water, and consequently the liquids in their body become increasingly concentrated. At the same time, we notice in the blood an increasingly pronounced hardening of the white blood cells, which depends on an arrest of these cells in the lymphatic pathways, as was verified during autopsies.
The histological examination of different organs of dogs that died from absolute insomnia demonstrated to me, in the most evident way, that the brain had undergone the greatest changes: a quantity of ganglia were in a state of fatty degeneration, the cerebral blood vessels were very often surrounded by a thick layer of white blood cells; one was tempted to say that the perivascular channels were filled with white blood cells, and in certain places, the blood vessels appeared as if compressed. Small capillary hemorrhages were encountered on the entire surface of the gray matter of the hemispheres, and larger hemorrhages around the optic nerves and in the substance of the optic lobes. The spinal cord appeared abnormally dry and anemic. The cardiac muscle was pale, the coronary vessels were filled with blood and contained, in most of these dogs, gas bubbles, which were also found in the large veins of the neck and in some cerebral vessels. The cardiac muscle fibers showed a finely granular degeneration. The spleen was in a state of hyperemia and appeared increased in volume, but I cannot prove it, as I did not make exact measurements. Another gap that I have left is that I did not observe the changes in the weight of different organs in dogs that died from insomnia.
I determined the weight of the dogs at the beginning of the experiment, then after their death; and in all cases, without exception, there was a weight loss, but it was not large and varied from 5% to 13%. As, in my life, I have been obliged to take part in experiments on starvation in different animals, I know very well the picture that animals that died of hunger present at autopsy; I know that the most surprising phenomenon in these animals is precisely the state of conservation of the brain, which loses the least of its weight and which preserves its normal state almost up to the moment of starvation where all the other organs and tissues of the body have already undergone profound changes and a more or less great loss of their weight. In animals that died of insomnia, on the contrary, we observe a diametrically opposed state, that is to say that, in them, the brain appears to be the site of predilection for the most profound and irreparable changes.
If my health permitted, I would very much like to undertake another series of experiments on the influence of insomnia on adult dogs and other animals; I would also try to obtain more exact data concerning the weight loss in relation to the different organs of the animal body.
But, however incomplete my experiments on absolute insomnia may be, they nevertheless provide us with conclusive proof of the profound importance of sleep for the organic life of animals with a cerebral system, and they also give us the right to consider as somewhat paradoxical, and even quite unfounded, the strange opinion that regards sleep as a useless, stupid and even harmful habit, as Girondeau does (5).
As communicated at the International Medical Conference in Rome, 1894
Marie De Manaceine, Sleep as one third of one’s lifetime, 1892 (Russian) Note: this book was later translated to English and became an absolute reference for Sleep science in the early 1900s. A digitisedPDF copy can be found here.
Renaudin, Observations on the pathological effects of insomnia (Annales medico-psychologiques, 1857)
Hammond. On Sleep. Gaillard’s Medical Journal, 1880 and Journal of Psychological medicine 1870
Girondeau. On brain circulation and its relationship with sleep. Paris 1868
These by Marie de Manacéïne were the first experiments to propose a vital function for sleep and to postulate that prolonged sleep deprivation would be lethal. These experiments were reproduced a few years later by Giulio Tarozzi (1898) and Lamberto Daddi (1899) on slightly older dogs. Daddi performed the sleep deprivation experiments and published the changes in metabolism and metabolites while Tarozzi published anatomical changes in the brain as seen through immunohistochemistry, on the same animals. Cesare Agostini also performed experiments of chronic sleep deprivation on a dog, observing death (1898) but adopted a different paradigm able to keep the animal awake through loud noises.
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
What is coccinella?
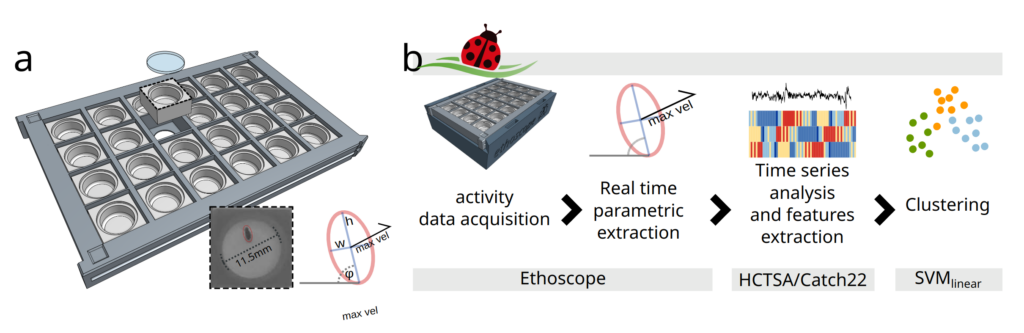
Coccinella is an innovative open-source framework developed for high-throughput behavioral analysis. Leveraging the power of distributed microcomputers, it facilitates real-time tracking of small animals, such as Drosophila melanogaster. Complementing this tracking capability, coccinella employs advanced statistical learning techniques to decipher and categorize observed behaviors. Unlike many high-resolution systems that often require significant resources and may compromise on throughput, coccinella strikes a balance, offering both precision and efficiency. Built upon the foundation of ethoscopes, this platform extracts minimalist yet crucial information from behavioral paradigms. Notably, in comparative studies, coccinella has demonstrated superior performance in recognizing pharmacobehavioral patterns, achieving this at a fraction of the cost of other state-of-the-art systems. This framework promises to complement current ethomics tools by providing a cost-effective, efficient, and precise tool for behavioral research. Coccinella analysis can be done in ethoscopy, a Python framework for analysis of ethoscope data.
How does it work?
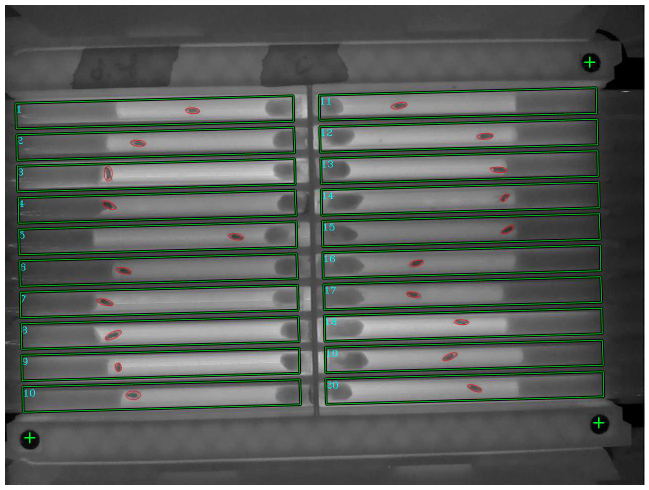
Coccinella uses ethoscopes to extract information about the activity of flies in real time. Ethoscopes are machines that use distributed computing via Raspberry PI to detect and interfere with behaviour. Given the off-the-shelf nature of the devices, the all setup is inexpensive and scales up very easily. As term of reference: our lab currently employs about 100 ethoscopes, with a processing power of 20 flies each.
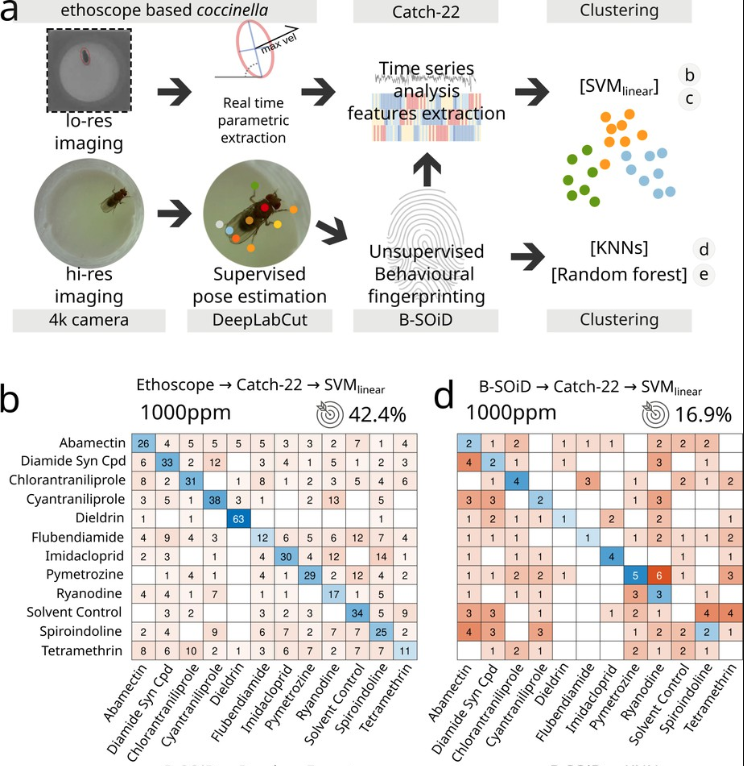
Data about the activity of the animal are then fed to a high-throughput toolbox for time series analysis called HCTSA or Catch22, initially developed at Imperial College London by our colleagues in the Maths Department. The toolbox performs numerous statistical tests aimed at segregating data in an unsupervised way and can therefore be used to cluster together data that the machine recognises as similar. In our case, we tried to identify which drugs have similar mode of action, potentially recognising and assigning the appropriate pharmacological pathways to new, uncharacterized compounds.
We also compared the performance of coccinella to state of the art systems and found that it performs even better!
This is important from the technical point of view but also from the standpoint of neuroscience because it shows that “less is more” when it comes to extracting and recognising behavioural data. In other words, you don’t need to carefully label posture and movement when characterising behaviour: reducing activity to its minimal terms actually works even better!
Joyce, M., Falconio, F.A., Blackhurst, L. et al. Divergent evolution of sleep in Drosophila species. Nat Commun15, 5091 (2024). https://doi.org/10.1038/s41467-024-49501-9
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
Elephants spend up to 18 hours a day eating grass, bushes, roots, shrubs to maintain their appropriate calorie intake. They sleep only 1 or 2 hours a day. Bats, on the other hand, are believed to sleep more than 20 hours a day. Finally, Great Frigatebird. They would normally sleep 9-10 hours a day and you would have hard time trying to get them to sleep less than that. Unless it’s migratory season. In that case, they sleep 40 minutes a day, while they flies for days and days in a row. Evolution is one of the great mysteries of sleep. Why do some animals require 20 hours, while others can cope with 1 or 2? Whatever sleep function is, how can it be accomplished in 10 hours in one season and 40 minutes in another, as it happens in migratory birds?
We won’t really understand what sleep is and what it does if we keep thinking about it in an anthropocentric way. We need to look at it from the evolutionary standpoint and only then we will be able to grasp what its role in nature is. This work marks our first big attempt in this direction. We did not compare sleep between elephants and bats. Too tricky to keep in the test tube and too evolutionary distant. Instead, we used seven species of Drosophila spanning an evolutionary distance of 5-50 Million years and with different ancestral origins and adaptation niches.
In all of them, we measure sleep using a computerised video tracking system based on Raspberry PIs which can be linked to robots to deliver sensory stimuli in real-time, such as puffs of air or automatic rotations of the test tube to keep them awake. We had actually used this device before to explore how fruitflies recognise and respond to salient stimuli during sleep. Here, we combined those with the excellent hidden Markov chain model initially proposed by the Griffith Lab at Brandeis and were able to confirm that different sleep stages as detected by the Markov chain do indeed coincide with different arousabilities. Deep sleeping flies are harder to wake up!
We found that all species sleep in more or less the same way, although for very different lengths of time. In almost all species, sleep is sexually dimorphic: females sleep only at night and males sleep in the afternoon too. Except for D. virilis: a cosmopolitan species believed to have arisen in the Miocene in the deserts of Afghanistan. Interestingly, this is something very recently found in other desert species too. You probably don’t want to be flying around in a desertic afternoon! So, sleep amount is generally conserved and obviously it adapts to species-specific ecological conditions, exactly as for the elephant and the bat. But what about sleep homeostasis? How do these exotic flies react when we try to keep them awake? For this, we turned to our trusty robots and kept flies awake for 24 hours in a row by rotating their little world around every time the fell asleep. A bit like in the Inception movie. Watch the first tube from the left to see the robot in action.
When you deprive an animal of sleep, it tries to recover some of it ASAP. This is a hallmark of sleep homeostasis and what we observed in D. melanogaster, but not in any of the other species! Like the migratory birds, they suddenly seemed OK not sleeping. No signs of tiredness. And even making our robot work for 7 days in a row – 168 hours – did nothing to them! These other species could stay awake just fine and showed no signs of tiredness. Except for melanogaster, which showed a steady increase in sleep pressure. However, at least some species were able to show rebound sleep when we used a different way of keeping them awake: social stress induced by male-male interaction in a laboratory boxing-ring equivalent. Stress can induce rebound sleep in many species, including rodents, and it does so by activating specific brain circuits as our colleagues recently showed.
Surprisingly, male-male interaction did lead to sleep rebound not just in melanogaster but also, simulans, sechelia, yakuba. Still no signs of homeostasis in the remaining three species though! What decides whether an animal will show homestasis? It seems the answer is in their brains. We found that, in general, sleep rebound correlated with an increase in synaptic strength. All the flies that showed rebound also showed a larger amount of a specific synaptic protein. And conversely, when we remove synaptic proteins from specific parts of the brain involved in learning and memory in D. melanogaster we get a similar effect: no tiredness after sleep deprivation.
We also go on and look at the evolution of pharmacology in these species and much more. Have a go at the manuscript yourself. It’s hopefully easy to read for everyone. hat is the take-home message? Well, we try to figure out what all this means in evolutionary terms. We think sleep has different functions in different species (doh!) and some functions therefore evolved for some species but not others. The one common thing all animals have in common is they all sit on the same planet which has been rotating at the same speed for a very long time. We believe this adaptation created sleep in the first place giving animals a chance to optimise their activities to days & nights. Then, other sleep functions kicked in. Some animals need sleep to cope with stress; some others need sleep to learn better; to memorize; to fight bacteria. Who knows how many different functions there are? Some need sleep for multiple reasons at once. This makes sense on multiple levels and can ultimately explain why elephants can do in 1 hour what bats seem to take 20 hours for!
Ethoscope-lab is a pre-baked Docker container featuring an installation of the multi user Jupyter Hub with Python and R kernels, ready to be used with Ethoscopy and Rethomics.
Why using ethoscope-lab?
Let me simply explain how we use it in our lab. We arranged a powerful workstation that acts as lab server and run a dockerized ethoscope-lab on it. The workstation has a local copy of all our ethoscope data (about 8 Terabyte as I type) and ethoscope-lab has local access on those, offering the quickest loading time. Users can then use their computer, or tablet to connect to the workstation and perform data analysis directly from the browser. The setup frees them from working at their desk and allows access to their data from anywhere in the world, guaranteeing at the same time the fastest computational performance even when they work on their laptops. Moreover, the system uses Jupyter notebook as default, meaning each analysis can be nicely annotated and exported to be shared with the world post-publication, along the original raw data.
To give a practical example: this series of repositories on zenodo contains the entire dataset of our latest paper (316Gb) and it’s paired to all the notebooks we used to generate each figure. Readers can download the dataset freely, install ethoscope-lab as docker container on any computer (irrespective of the operating system they adopt) and reproduce all our analyses!
On 29 September 2021 by Giorgio With 0 Comments
- papers
An AI generated podcast explaining the paper in a fun and engaging way (created with Google’s NotebookLM)
One of the most puzzling aspects of sleep is that it cannot happen without depriving us of our full conscious experience. Whatever the function of sleep is, it cannot be achieved without disconnecting our brains from the external world. A full conscious state and sleep are not compatible, it seems, to the point that one of the definitions of consciousness is that “it is all that fades away when we are in dreamless sleep”.
The fact that the brain has to surrender to the tyranny of sleep is also the main reason why scientists believe (in a rather dogmatic fashion) that sleep is “of the brain, by the brain for the brain“. Yet, even during sleep parts of our brains retain some ability to process external information. In the 1960s, Oswald et al formally showed that sleeping humans could wake up in response to some salient stimuli, such as their names being called, but not in response to stimuli of identical strength but no salience, such as other people’s names or their names played in reverse.
This finding has been confirmed and extended over the decades in the scientific literature, providing evidence that it applies to even more complex nuances of saliency, such as an angry tone of voice. The videos below suggest that scientific literature is certainly less comprehensive and (less amusing) than the phenomenon in its entirety.
Pets wake up to food odours and food-related noises.And the human brain is certainly able of very deep sensory processing!
Even though we have numerous scientific and anecdotal evidence that animals and humans can wake up to salient sensory stimuli during sleep, hardly anything is known about the biological underpinning of this phenomenon. And here: enter Drosophila melanogaster! What better animal model than flies to dissect this amazing brain property?
In a paper titled “Sensory processing during sleep in Drosophila melanogaster” published in Nature, we introduce flies as the ideal animal model to dive into the biology of how a brain can simultaneously be asleep and respond to external stimuli.
Postdoc Alice French took the lead on this amazing project to show that even flies can recognise salient stimuli in their sleep and react accordingly, modulating their response based on their internal state. We initially expanded the robotic platform we had previously built in the lab, called ethoscopes, which allows us to monitor and interfere with flies using inexpensive @Raspberry_Pi computers. Alice wanted to build a robotic component able to challenge single flies with specific odour but only while they were asleep, to record whether they would wake up or not. She obviously started with…. LEGO!
In our first prototype, we built a robot able to operate a LEGO valve so to send a puff of air to the sleeping fly. LEGO valves were a good start because we needed 500 of them.
The system worked and we went from those early all-LEGO prototypes (left) to the final 3D printed product (right).
Using this ethoscope module we could challenge sleeping flies with different odours and check whether they would respond differently to some of them. We found they did! Flies would respond to 5% acetic acid for instance, but not to 10% acetic acid. Not only that, the valence of the odour could be modulated by internal states. Flies that had received a little starvation were increasing their response specifically to food-related odours. When we gave alcohol to flies, on the other hand, we found drunk Drosophilae were less responsive to odours in general showing somehow a deeper sleep state.
Now, flies are arguably the best animal model to study circuit neuroscience these days. We have a full connectome of the fly brain and countless genetic tools that allow us to turn neurons on and off. So that is what we did. We started turning neurons on and off in the fly brain, looking for some that would modulate their ability to sense stimuli during sleep. We found them!
We actually found the whole circuit, connecting the “fly nose” all the way to the sleep centers in the brain. And when we used thermogenetics to switch those neurons on or off with infrared radiation, we could interfere with that process and make the flies more or less responsive.
In short, we have shown that flies can recognise and respond to odours during sleep, waking up only to those that they consider salient. We also show that this phenomenon is plastic and modulated by internal states, with animals being more likely to wake to food odours after a little starvation. We also described a blueprint for a neuronal circuit that connects the peripheral olfactory receptor neurons all the way to known sleep-regulating centres in the fly brain. We explore three prototypical gate-points that modulate subconscious processing of olfactory information during sleep: two at the periphery and one in the central brain.
The story is important and of general interest for at least three reasons:
for the groundbreaking implications it has on the consciousness field, introducing flies as a model to study subconscious processing of information, and providing an experimental paradigm that allows to empirically face some key questions of the field;
for the implications it has on the sleep community, describing the neuronal circuit regulating sensory processing during sleep, a neuronal feature that is poorly understood in any other animal model. Our description of the circuit regulating sensory processing during sleep is the most accurate to date and the work also potential future medical significance, for instance in the study of altered states of consciousness, such as coma;
for the implications it has on the larger neuroscience community, describing how a circuit modulates the processing of sensory information to distinguish valence.
Drosophila has been employed to study arousal threshold many times before. There are many studies in which flies can be used to gauge sleep “depth” by using quantitative mechanical stimuli, such as simple vibration or touch. Our study is the first one to study a more puzzling property: how do we recognise qualitative stimuli during sleep? How do we recognise our own name while unconscious?
The video abstract below provides more information on the contents and the implications of the work.
Drosophila melanogaster, commonly known as fruit fly or more appropriately vinegar fly, is the second most common animal model used in research. Initially established by Thomas Hunt Morgan at the beginning of 1900s to provide an empirical base to the groundbreaking hypotheses of Darwin, flies have contributed to science in every realm, from development to genetics and neuroscience. 6 Nobel prizes have been awarded to flies in the past century, with the last one being awarded in 2018 to three Drosophila researchers for their work in the characterisation of circadian behaviour.
My laboratory uses flies to try and answer one simple, yet fascinating question: why do we sleep? What is sleep for and why humans and all animals seem to require sleep? Our approach is somehow different mainstream one, because flies force us to think to the problem in an unusual and more creative way. So far this has paid off egregiously, and we have managed to make very important discoveries that apply well beyond the fly realm.
One aspect of our research that may be particularly interesting for someone puzzled about the science of physical well being, is that we do not consider sleep to be a prerogative of the brain but actually a phenomenon that affects every part of our body. Whenever we lack sleep – whether for fun or for work – we can feel an effect of sleep deprivation not just on our cognitive performance but on our very body too. This is more than a subjective feeling: it is a well-established phenomenon in humans and animals. Why is it so? Studying sleep deprivation in flies we hope to give an answer to this question.
In particular, we use state of the art technology to a) deprive flies of sleep employing custom-made robots and b) exploring what changes at the cellular level when we lack sleep. How genes, proteins, and other molecules change their composition when we lack sleep?
We can use the same robotic technology to also study physical behaviour in these animals: are they in good shape? Can they climb a wall as they normally do? Can they fly with the same stamina and precision? A great amount of literature in the field of muscular degeneration has been obtained in fruit flies and we have learned a great deal about genes controlling these aspects and how they fail in disease.
A very important corollary of our research is that understanding the functions of sleep opens the door to what we somehow half-jokingly call “the sleep pill”. If could understand what aspects of sleep make us refreshed and performing – both behaviourally and physically – we could then replace sleep pharmacologically. Or we could consolidate the beneficial aspects of sleep to increase its restorative power. To do that, we first need to understand what sleep is and what it does.
What would we do with a philanthropic donation?
We would employ the money to retain a brilliant young research assistant for a year or longer so that she could continue working on her project. The student recently graduated from an MSci in Neuroscience and she joined our laboratory for a summer placement in order to gain first-hand insights into our research. If she could stay longer, she could join and potentiate the research line of the laboratory that looks at the direct consequences of sleep deprivation. I have been working with Imperial Alumni who were kind enough to donate to my laboratory in the past. It has been a great honour and a pleasure and I am looking forward to doing this again.